Here, we present a Cas9-based exon23 deletion protocol to restore dystrophin expression in iPSC from Dmdmdx mouse-derived skin fibroblasts and directly differentiate iPSCs into myogenic progenitor cells (MPC) using the Tet-on MyoD activation system.
A subscription to JoVE is required to view this content. Sign in or start your free trial.
Method Article
CRISPR/Cas9 Technology in Restoring Dystrophin Expression in iPSC-Derived Muscle Progenitors
In This Article
Summary
Abstract
Duchenne muscular dystrophy (DMD) is a severe progressive muscle disease caused by mutations in the dystrophin gene, which ultimately leads to the exhaustion of muscle progenitor cells. Clustered regularly interspaced short palindromic repeats/CRISPR-associated 9 (CRISPR/Cas9) gene editing has the potential to restore the expression of the dystrophin gene. Autologous induced pluripotent stem cells (iPSCs)-derived muscle progenitor cells (MPC) can replenish the stem/progenitor cell pool, repair damage, and prevent further complications in DMD without causing an immune response. In this study, we introduce a combination of CRISPR/Cas9 and non-integrated iPSC technologies to obtain muscle progenitors with recovered dystrophin protein expression. Briefly, we use a non-integrating Sendai vector to establish an iPSC line from dermal fibroblasts of Dmdmdx mice. We then use the CRISPR/Cas9 deletion strategy to restore dystrophin expression through a non-homologous end joining of the reframed dystrophin gene. After PCR validation of exon23 depletion in three colonies from 94 picked iPSC colonies, we differentiate iPSC into MPC by doxycycline (Dox)-induced expression of MyoD, a key transcription factor playing a significant role in regulating muscle differentiation. Our results show the feasibility of using CRISPR/Cas9 deletion strategy to restore dystrophin expression in iPSC-derived MPC, which has significant potential for developing future therapies for the treatment of DMD.
Introduction
Duchenne muscular dystrophy (DMD) is one of the most common muscular dystrophies and is characterized by the absence of dystrophin, affecting 1 of approximately 5,000 newborn boys worldwide1. Loss of dystrophin gene function results in structural muscle defects leading to progressive myofibers degeneration1,2. Recombinant adeno-associated virus (rAAV)-mediated gene therapy system has been tested to restore the dystrophin expression and improve muscle function, such as gene replacement using micro-dystrophins (µ-Dys). However, the rAAV approach requires repeated injections to sustain expression of the functional protein3,4. Therefore, we need a strategy that can provide effectively and permanently recover dystrophin gene expression in patients with DMD. The Dmdmdx mouse, a mouse model for DMD, has a point mutation in exon 23 of the dystrophin gene that introduces a premature termination codon and results in a non-functional truncated protein lacking the C-terminal dystroglycan binding domain. Recent studies demonstrated the use of CRISPR/Cas9 technology to restore dystrophin gene expression by accurate gene correction or mutant exon deletion in small and large animal5,6,7. Long et al.8 reported the method for correcting the dystrophin gene mutation in Dmdmdx mouse germline by homology-directed repair (HDR) based CRISPR/Cas9 genome editing. El Refaey et al.9 reported that rAAV could efficiently excise the mutant exon 23 in dystrophic mice. In these studies, gRNAs were designed in the introns 20 and 23 to cause double-stranded DNA breaks, which partially restored the dystrophin expression after DNA repair via non-homologous end joining (NHEJ). Even more exciting, Amoasii et al.10 recently reported the efficacy and feasibility of rAAV-mediated CRISPR gene editing in restoring dystrophin expression in canine models, an essential step in future clinical application.
DMD also causes stem cell disorders11. For muscle damage, residential muscle stem cells replenish dying muscle cells after muscle differentiation. However, the consecutive cycles of injury and repair lead to shortening of telomeres in muscle stem cells12, and premature depletion of stem cell pools13,14. Therefore, a combination of autologous stem cell therapy with genome editing to restore dystrophin expression can be a practical approach for treating DMD. The CRISPR/Cas9 technology provides the possibility of generating autologous genetically corrected induced pluripotent stem cells (iPSC) for functional muscle regeneration and prevent further complications of DMD without causing immune rejection. However, iPSCs have a risk of tumor formation, which could be alleviated by the differentiation of iPSC into myogenic progenitor cells.
In this protocol, we describe the use of non-integrating Sendai virus to reprogramming dermal fibroblasts of Dmdmdx mice into iPSCs and then recover dystrophin expression by CRISPR/Cas9 genome deletion. After validation of Exon23 deletion in iPSC by genotyping, we differentiated genome-corrected iPSC into myogenic progenitors (MPC) via MyoD-induced myogenic differentiation.
Access restricted. Please log in or start a trial to view this content.
Protocol
All animal handling and surgical procedures were performed by a protocol approved by the Augusta University Institutional Animal Care and Use Committee (IACUC). Mice were fed standard diet and water ad libitum.
1. Isolation of primary mouse fibroblasts from adult Dmdmdx mice
- Euthanize adult Dmdmdx mice (male, 2 months old) by CO2 asphyxiation and thoracotomy according to IACUC approved by Medical College of Georgia, Augusta University. Cut the tail with a sterile scalpel in a sterile condition under the laminar hood. Rinse the tail with 70% ethanol for 5 min, and then wash with sterile phosphate-buffered saline (PBS) in a 6 cm dish.
- Peel the tail skin off by a sharp incision from the base to the tail tip along the tail skin, and then gently peel off the tail skin with tweezers. Mince the skin to a size of 1 mm3 using a sterile scalpel and move the minced skin tissue to a 6 cm dish in Dulbecco’s minimal essential medium/Ham’s F12 (DMEM/F12) containing 0.1% collagenase IV and 1 U/mL of dispase.
- Digest the skin tissue in a culture dish for 2 h at 37 °C in a 5% CO2 incubator.
- Coat a 6-well plate with fibronectin and 0.2% gelatin (1 mL of fibronectin in 199 mL of 0.2% gelatin; Table of Materials) and incubate at 37 °C for 1 h.
- Dissociate the digested skin tissue with a 1 mL pipet tip and transfer the tissue and supernatant to a sterile 15 mL conical centrifuge tube. Centrifuge at 217 x g for 3 min at room temperature, discard the supernatant and resuspend the pellet in 1.5 mL of fibroblast medium (Table of Materials).
- Culture the pellets including incomplete digested skin tissue from step 1.5 on the 6-well plate coated with fibronectin and 0.2% gelatin from step 1.4 in a 37 °C, 5% CO2 incubator. Replace the medium 24 h after the initial plating to remove unattached cells, and change the medium every 48 h.
2. Reprogramming mouse skin fibroblasts into iPSCs
- Two days before transduction, digest mouse dermal fibroblasts from step 1.6 with the cell detachment solution (Table of Materials) in a 37 °C incubator with a humidified atmosphere of 5% CO2 for 5 min.
- Count cells using a hemacytometer and centrifuge at 217 x g for 3 min.
- Seed cells at a density of 1−2 x 10⁵ cells per well onto a 6-well plate and culture with fibroblast medium (Table of Materials) in a 37 °C incubator with a humidified atmosphere of 5% CO2.
- On the day of transduction (day 0), estimate the cells and calculate the volume of each virus required to reach the target multiplicity of infection (MOI) of 5, 5, and 3 (i.e., KOS MOI = 5, hc-Myc MOI = 5, hKlf4 MOI = 3) according to the commercial manual.
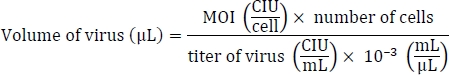
- Thaw three Sendai tubes in a 37 °C water bath for 5−10 s and add the calculated volumes of each of the three Sendai tubes to 1 mL of fibroblast medium (Table of Materials).
- Remove the fibroblast medium from step 2.3 and add the reprogramming virus mixture to the wells containing the cells. Incubate the cells overnight in a 37 °C incubator with a humidified atmosphere of 5% CO2.
- Replace the medium with fresh fibroblast medium 24 h after transduction. Culture the cells for one week with medium exchange every other day.
- Harvest infected mouse fibroblasts on day 7 after transduction with 0.05% trypsin/EDTA and place on dishes that are previously coated with fibronectin and 0.2% gelatin.
- Culture the infected mouse fibroblasts from step 2.6 with complete mouse embryonic stem cell (ES) growth medium (Table of Materials) in a 37 °C incubator with a humidified atmosphere of 5% CO2 and change medium daily.
- From the 8th day, observe the plate under an inverted microscope every other day to identify the appearance of cell clumps with the morphology of mouse ES.
3. Using alkaline phosphatase live stain and flow cytometry to quantify reprogramming efficiency
- Remove the culture media from each well and rinse with DMEM/F-12 for 2−3 min.
- Apply 2 mL of 1x alkaline phosphatase (AP) live stain working solution (1:500 dilution in DMEM/F-12) to the adherent cells, and incubate in a 37 °C incubator with a humidified atmosphere of 5% CO2 for 30 min.
- Aspirate the AP live stain and wash twice with PBS for 5 min each.
- Digest the cells with the cell detachment solution (Table of Materials) in a 37 °C incubator with a humidified atmosphere of 5% CO2 for 5 min. Perform flow cytometry to determine the reprogramming efficiency.
4. Selecting and harvesting ES-like cells
- Examine the colonies from step 2.8 under an inverted microscope.
- Mark the colonies at the bottom of the dish with a self-inking object marker.
- Apply greased cloning rings to cover the marked cell colonies. Add 100 μL of 0.05% trypsin/EDTA to each cloning ring at 37 °C for 5 min, and then transfer the digested cells with 100 μL pipette tips to 48-well culture plates containing mES growth medium.
- Incubate the cells in 48-well culture plates in a 37 °C incubator with a humidified atmosphere of 5% CO2. Passage the cells to 6 cm dish when they reach 70% confluence.
- Repeat steps 4.3 and 4.4 for several times until uniform dorm-shaped clones are obtained.
5. Freezing iPSCs for cryopreservation
- Dissociate the selected iPSCs from step 4.5 with trypsin, versene, and chick plasma (TVP; Table of Materials) solution at 37 °C in a 5% CO2 incubator for 30 min.
- Collect the cells in a sterile 15 mL conical tube and centrifuge at 217 x g for 3 min at room temperature.
- Aspirate the supernatant and re-suspend the cell pellet in 2 mL of mouse ES frozen medium (Table of Materials) to obtain 1 mL per cryovial.
- Add cells to cryovials and freeze using a freezer container that provides the critical, repeated -1 °C/min cooling rate required for cryopreservation at -80 °C overnight.
- Transfer frozen vials into a liquid nitrogen tank.
6. Immunofluorescence staining for stem cell markers in iPSCs
- Seed iPSCs from step 5.1 cultured with mES medium into an 8-well chamber slide coated with poly-D-lysine/laminin (Table of Materials) at the appropriate density to achieve between 1−2 x 10⁴ cells per well and incubate in a 37 °C incubator with a humidified atmosphere of 5% CO2 for 48 h.
- Immerse the slides in 4% formaldehyde for 15 min at room temperature, and then immerse the slides in PBS twice for 5 min each time.
- Incubate sections with a mouse IgG-blocking reagent (Table of Materials), and 5% goat serum for 1 h at room temperature.
- Dilute the primary antibodies in protein diluent (mouse-anti-SSEA1, 1:100, rabbit-anti-Nanog, 1:500; rabbit-anti-POU class 5 homeobox 1 [OCT4], 1:500; rabbit-anti-SRY-box 2 [SOX2], 1:500; rabbit-anti-Lin-28 homolog A [Lin28A], 1:400) (Table of Materials). Apply antibodies to the cells and incubate at 4 °C overnight in a humidified chamber.
- Discard the primary antibody solution and wash the slides 3x in PBS.
- Apply second antibodies (Alexa488-conjugated goat-anti-mouse antibody and Alexa555-conjugated goat-anti-rabbit, 1:400 each) in M.O.M. protein diluent on slides and incubate for 45 min at room temperature.
- Wash the slides 3x in PBS and mount sections with mounting medium containing 4’6-diamidino-2-phenylindole (DAPI).
- Take pictures with a confocal microscope.
7. Investigating the pluripotency of iPSCs in vivo
- Dissociate the iPSCs from step 5.1 into single cells using TVP solution in a 37 °C incubator with a humidified atmosphere of 5% CO2 for 30 min.
- Count cells using a hemacytometer and centrifuge at 217 x g for 3 min.
- Aspirate the supernatant and resuspend the pellet with mES medium in a 1.5 mL sterile centrifuge tube at a concentration of 5 x 10⁵ cells/30 μL for cell transplantation.
- Remove hair from both hind limbs of immunodeficient mice using hair clippers.
- Anesthetize mice with ketamine (100 mg/kg) and clean the injection site with 75% alcohol.
- Inject 30 μL of iPSC suspension from step 7.3 intramuscularly into the gastrocnemii, using a 31 G needle.
- Two weeks after the injection, harvest the mouse gastrocnemii and embed in optimal cutting temperature (OCT) compound, snap freeze and cut into 5-μm sections15,16.
- Fix sections in 4% formaldehyde for 15 min at room temperature, and then wash the slides twice in PBS for 5 min each time.
- Block the cells with 5% goat serum protein diluent for 1 h at room temperature.
- Add diluted primary antibody (rabbit anti-AFP, 1:50; rabbit anti-SMA, 1:50; rabbit anti-TH, 1:50) to the slides and incubate at 4 °C overnight in a humidified chamber.
- Discard the primary antibody solution, wash the cells 3x (5 min/wash) in PBS, add a 1:400 diluted Alexa555-conjugated goat-anti-rabbit antibody to slides, and incubate for 45 min at room temperature.
- Wash slides 3x (5 min/wash) in PBS, and mount sections with mounting medium containing DAPI.
8. Construction of CRISPR/Cas9 lentiviral vector targeting introns flanking dystrophin exon 23
- Design two pairs of gRNA oligos targeting intron-flanked dystrophin exon 23 via http://crispor.tefor.net/crispor.py.
NOTE: The designed pairs are as follows:
i22sense: 5’-CACCGTTAAGCTTAGGTAAAATCAA- 3’
i22anti-sense: 5’-AAACTTGATTTTACCTAAGCTTAAC-3’
i23sense: 5’-CACCGAGTAATGTGTCATACCTTCT- 3’
i23anti-sense: 5’-AAACAGAAGGTATGACACATTACTC-3’). - Digest and dephosphorylate 5 µg of lentiviral CRISPR plasmid (lenti-CRISPRv2-blast [a gift from Mohan Babu] and lenti-Guide-Hygro-iRFP670 [a gift from Kristen Brennand]) (Table of Materials) with BsmB1/Esp3I for 30 min at 37 °C. For 5 µg of plasmids, add 3 µL of BsmB1 restrict enzyme, 3 µL of fast alkaline phosphatase, 6 µL of 10x enzyme digest buffer and 0.6 µL of 100 mM DTT in 60 µL reaction).
- Load the reactions onto a 0.8% agarose gel. Run the gel at 100−150 V for 30 min.
- Purify digested plasmid in-gel using a gel extraction kit (Table of Materials) and elute in 20 µL of H2O.
- Phosphorylate and anneal each pair of the gRNA oligonucleotides containing 1 µL of each oligonucleotide at 100 µM, 1 µL of 10x T4 ligation buffer, 0.5 µL of T4 polynucleotide kinase (PNK), 6.5 µL of ddH2O at 37 °C for 30 min, and then 95 °C for 5 min and then ramp down to 25 °C at 5 °C/min.
- Ligate a 1:200 dilution of the annealed gRNA oligonucleotides into the plentiCRISPR V2-Blast or plentiGuide-Hygro-iRFP670. Mix 50 ng of BsmB1/Esp3I digested vectors with 1 µL of diluted oligo duplex and 5 µL of 2x ligase buffer plus 1 µL of ligase in a 11 µL reaction system and incubate for 10 min at room temperature.
- Perform transformation with 3 µL of ligation product into 50 µL competent cells (Table of Materials) according to the manufacturer’s instructions.
- Spread the transformed competent cells in an agar plate with 100 µg/mL carbenicillin and incubate at 31.5 °C for 18 h.
- Pick colonies with 10 µL sterile pipette tips and culture in 5 mL of terrific broth (Table of Materials) containing 100 µg/mL carbenicillin at 31.5 °C, 185 rpm in a shaker incubator for 21 h.
- Purify the plasmid DNA using the mini-prep and midi-prep kits (Table of Materials).
- Verify the mini-prep plasmids by restriction digestion. For the 20 µL reaction system, add 1 µg of plasmid DNA, 2 µL of digest reaction buffer (Table of Materials) and 1 µL of restriction enzyme mixture (0.5 µL of KpnI-HF and 0.5 µL of AgeI-HF for plentiCRISPR V2-Blast-i22; 0.5 µL of NotI-HF and 0.5 µL of EcoRI-HF for plentiGuide-Hygro- iRFP670- i23). Incubate the reaction system for 1 h at 37 °C.
- Load the reactions onto a 0.8% agarose gel. Run the gel at 100−150 V for 30 min.
NOTE: The correct bands for plentiCRISPR V2-Blast-i22 should be 622 bp and 12.2 kb, and the correct bands for plentiGuide-Hygro- iRFP670- i23 should be 2.6 kb and 7.1 kb.
9. Lentiviral vector packaging
- Culture 7 x 10⁵ 293FT cells in 5 mL of DMEM media containing 10% fetal bovine serum in a 6 cm dish overnight at 37 °C, 5% CO2.
- Prepare a cocktail (1 µg of plentiCRISPR V2-Blast-i22 or plentiGuide-Hygro-iRFP670-i23, 750 ng of psPAX2 packaging plasmid, 250 ng of pMD2.G envelope plasmid, and 5 µL of transfection reagent A [Table of Materials] in 100 µL of reduced serum MEM media).
- Prepare a mixture of 5 µL of transfection reagent B (Table of Materials) in 100 µL of reduced serum MEM media.
- Add 100 µL of transfection reagent B mixture to plasmid mixture from step 9.2 and incubate for 5 min at room temperature.
- Add the DNA-lipid complex (from step 9.4) dropwise to the 293FT cells. Incubate overnight at 37 °C with 5% CO2.
- Add virus production enhancer (500x) (Table of Materials) to each dish the next day and incubate for 24 h at 37 °C, 5% CO2.
- Collect medium from cells using pipettes on the next two days and filter the medium through a 0.45 µm filter to remove the cells.
10. Concentration and purification of lentiviral vectors
- Precipitate lentiviral vector in the medium of step 9.7 overnight at 4 °C with 5x polyethylene glycol 4000 (PEG4000, 8.5% final concentration) and 4 M NaCl (0.4 M final concentration).
- Centrifuge the viral media containing the PEG4000 solution at 2,095 x g and 4 °C for 30 min, remove and discard the supernatant.
- Resuspend the pellets with 500 µL of serum reduced MEM media (lentivirus titer: lenti-CRISPR V2-gRNAi22: 1.56 x 10⁸, lenti-iRFP670-gRNAi23: 1.3 x 10⁸, lenti-CRISPR V2-control: 3.13 x 10⁷, lenti-iRFP670-control: 5.9 x 10⁷). Store at -80 °C until use.
11. Deletion of exon 23 in mouse iPSCs with two guide RNAs (gRNAs) coupled with Cas9
- Plate the mouse iPSCs from step 4.5 in a 24-well plate coated with fibronectin and gelatin.
- After the cells reach 50% confluence, switch to the fresh culture medium (complete mouse embryonic stem cell growth medium) containing 8 µg/mL polybrene).
- Add 100 µL of the lentiviral particle solution from step 10.3 including lenti-CRISPR V2-gRNAi22, lenti-iRFP670-gRNAi23 and control (empty vector: lenti-CRISPR V2, lenti-iRFP670) to mouse iPSCs. Incubate cells for 3 days at 37 °C with 5% CO2.
- Select stably infected cells with media containing 2.5 µg/mL blasticidin and 100 µg/mL hygromycin B by determining the minimum concentration of blasticidin and hygromycin B required to kill the un-infected cell.
NOTE: Un-infected cells would be killed by blasticidin and hygromycin B. - Digest the selected mouse iPSCs with 0.5 mL of TVP solution each well (24-well plate) and incubate cells for 30 min at 37 °C with 5% CO2.
- Dissociate the iPSCs into single cells by pipetting, count cells with a cell counting chamber and then dilute about 150 digested single cells with mES medium into 10 cm dish for culture at 37 °C with 5% CO2.
- After about 10 days, pick single colonies under an inverted microscope using 10 µL sterile pipette tips (96 colonies need to be picked).
- Transfer the picked colonies into 50 µL of TVP solution each well (96-well plate, one colony each well), digest at 37 °C for 30 min, and then seed the digested cells into two 96-well culture plates to keep culture (one for genotyping).
- Incubate in a CO2 incubator at 37 °C until 70% confluent.
12. Identification of iPSC colonies with exon23 deletion
- Remove the medium in 96-well plate when the cell colonies reach 70% confluence.
- Add 25 µL of lysis reagent (Table of Materials) containing proteinase K solution (1 mL of proteinase K in 100 mL of lysis reagent) to each well, and transfer the lysate to a 96-well PCR plate.
- Seal the PCR plate and incubate the plates at 55 °C for 30 min, and then at 95 °C for 45 min to lyse the cells and denature the proteinase K.
- Carry out PCR reaction with 2 µL of lysate from step 12.3. For the 20 µL PCR reaction, add 2 µL of lysate, 10 µL of 2x DNA polymerase premix (Table of Materials), 7 µL of DNase-free water, and 1 µL of DMD exon 23 primers (Table 1).
- Use the following parameters for PCR reaction: 98 °C for 1 min, 35 cycles of 98 °C for 10 s, 60 °C for 15 s, 72 °C for 30 s, and a final extension at 72 °C for 1 min.
- Load the PCR reaction onto a 2% agarose gel. Run the gel at 100−150 V for 30 min.
- Inspect the gel under UV light (the knockout efficiency is 3/94).
13. Using the Tet-on MyoD activation system to directly differentiate iPSC into myogenic progenitor cells (MPC)
- Package the LV-TRE-VP64-mouse MyoD-T2A-dsRedExpress2 and LV-TRE-VP16 mouse MyoD-T2A-dsRedExpress2 (a gift from Charles Gersbach) (Table of Materials) as previously described for lenti-CRISPRv2-blast and lenti-gRNA-iRFP670 vectors in sections 9 and 10.
- Infect mouse iPSC with lentivirus-TRE-VP64-MyoD-T2A-dsRed-Express2 or lentivirus-TRE-VP16-MyoD-T2A-dsRedExpress2 as previously described for lenti-CRISPRv2-blast and lenti-gRNA-iRFP670 vectors in steps 11.1−11.3.
- Select cells with 1 μg/mL puromycin after three days of infection to obtain a pure transduced cell population.
- Add 3 μg/mL doxycycline into culture media (10% FBS DMEM) to MPC differentiation. Replace fresh medium supplemented with doxycycline every two days.
14. Quantitative reverse transcription PCR for evaluating dynamic muscle differentiation and DMD exon 22-24 expression
- Extract cellular RNA after 0, 3, 6, and 10 days after doxycycline treatment using RNA isolation reagent, reversely transcribe RNA into cDNA by using first strand cDNA synthesis kit (Table of Materials).
- For the 20 µL qPCR reaction system, add 1 µL of cDNA, 10 µL of PCR reaction buffer (Table of Materials), 8 µL of DNA H2O, and 1 µL of mixture of forward and reverse primers (glyceraldehyde-3-phosphate dehydrogenase [GAPDH], skeletal muscle [ACTA1], OCT4 and DMD exon22, DMD exon23, and DMD exon24, see Table 1).
- Use the following parameters for PCR reaction: 50 °C for 2 min, 95 °C for 2 min, 40 cycles of 95 °C for 15 s, 60 °C for 1 min, melt curve 65.0 °C to 95.0 °C, increment 0.5 °C.
15. Immunofluorescence staining of myosin heavy chain 2 (MYH2) and dystrophin protein expression
- Plate doxycycline-induced, lenti-TRE-MyoD modified cells from step 13.4 onto 8-well culture slides.
- Fix cells in 4% formaldehyde for 15 min at room temperature, and then wash the slides twice in PBS for 5 min each time.
- Block the cells with 5% goat serum protein diluent for 1 h at room temperature.
- Add rabbit-anti-dystrophin antibody (1:300) and mouse-anti-MYH2 antibody (1:100) to the slides, incubate at 4 °C overnight in a humidified chamber.
- Discard the primary antibody solution, wash the cells 3x (5 min/wash) in PBS, add 1:400 diluted Alexa488-conjugated goat-anti-rabbit antibody and Alexa555-conjugated goat-anti-mouse antibody to slides, and incubate for 45 min at room temperature.
- Wash the slides 3x (5 min/wash) in PBS, and mount sections with mounting medium containing DAPI.
Access restricted. Please log in or start a trial to view this content.
Results
Establishment of Dmdmdx skin fibroblasts derived iPSC. We demonstrated the efficiency of generating mouse iPSCs from Dmdmdx mice derived skin fibroblast using the integration-free reprogramming vectors. Figure 1A demonstrated that the appearance of embryonic stem cell (ESC)-like colonies at three weeks after infection. We evaluate the efficiency of iPSC induction by live alkaline phosphatase (AP) stain; Figure 1B s...
Access restricted. Please log in or start a trial to view this content.
Discussion
Duchenne Muscular Dystrophy (DMD) is a destructive and ultimately fatal hereditary disease characterized by a lack of dystrophin, leading to progressive muscle atrophy1,2. Our results demonstrate the restored dystrophin gene expression in Dmdmdx iPSC-derived myogenic progenitor cells by the approach of CRISPR/Cas9-mediated exon23 deletion. This approach has three advantages.
First, we generated iPSCs from Dmdmdx m...
Access restricted. Please log in or start a trial to view this content.
Disclosures
The authors have nothing to disclose.
Acknowledgements
Tang and Weintraub were partially supported by NIH-AR070029, NIH-HL086555, NIH-HL134354.
Access restricted. Please log in or start a trial to view this content.
Materials
| Name | Company | Catalog Number | Comments |
|---|---|---|---|
| Surgical Instruments | |||
| 31-gauge needle | Various | ||
| Sharp Incision | Various | ||
| Sterile Scalpels | Various | ||
| Tweezers | Various | ||
| Fibroblast medium (for 100 mL of complete medium) | Company | Catalog Number | Volume |
| 2-Mercaptoethanol (55 mM) | Gibco | 21-985-023 | 0.1 mL |
| Antibiotic Antimycotic Slution 100x | CORNING | MT30004CI | 1 mL |
| Dulbecco's Modified Eagle's Medium - high glucose | SIGMA | D6429 | 87 mL |
| Fetal Bovine Serum Characterized | HyClone | SH30396.03 | 10 mL |
| L-Glutamine solution | SIGMA | G7513 | 1 mL |
| MEM Non-Essential Amino Acids Solution (100x) | Gibco | 11140076 | 1 mL |
| TVP solution (for 500 mL of complete solution) | Company | Catalog Number | Volume |
| Chicken Serum | Gibco | 16110-082 | 5 mL |
| EDTA | Sigma-Aldrich | E6758 | 186 mg |
| Phosphat-buffered saline | to 500 mL | ||
| Trypsin (2.5%) | Thermo | 15090046 | 5 mL |
| mES growth medium(for 500 mL of complete solution) | Company | Catalog Number | Volume |
| 2-Mercaptoethanol (55 mM) | Gibco | 21-985-023 | 0.5 mL |
| Antibiotic Antimycotic Slution 100x | CORNING | MT30004CI | 5 mL |
| Dulbecco's Modified Eagle's Medium - high glucose | SIGMA | D6429 | 408.5 mL |
| Fetal Bovine Serum Characterized | HyClone | SH30396.03 | 75 mL |
| L-Glutamine solution | SIGMA | G7513 | 5 mL |
| Mouse recombinant Leukemia Inhibitory Factor (LIF), 0.5 x 10⁶ U/mL | EMD Millipore Corp | CS210511 | 500 μL |
| MEK/GS3 Inhibitor Supplement | EMD Millipore Corp | CS210510-500UL | 500 μL |
| MEM Non-Essential Amino Acids Solution (100x) | Gibco | 11140076 | 5 mL |
| The ES cell media should not be stored for more than 4 weeks and with inhibitors not more than 2 weeks. | |||
| mES frozen medium(for 50 mL of complete solution) | Company | Catalog Number | Volume |
| Dimethyl sulfoxide (DMSO) | SIGMA | D2650 | 5 mL |
| Dulbecco's Modified Eagle's Medium - high glucose | SIGMA | D6429 | 24.9 mL |
| Fetal Bovine Serum Characterized | HyClone | SH30396.03 | 25 mL |
| Mouse recombinant Leukemia Inhibitory Factor (LIF), 0.5 x 10⁶ U/mL | EMD Millipore Corp | CS210511 | 50 μL |
| Name of Material/ Equipment | Company | Catalog Number | RRID |
| 0.05% Trypsin/0.53 mM EDTA | CORNING | 25-052-CI | |
| 4% Paraformaldehyde | Thermo scientific | J19943-k2 | |
| Accutase solution | SIGMA | A6964 | Cell detachment solution |
| AgeI-HF | NEB | R3552L | |
| Alexa488-conjugated goat-anti-mouse antibody | Invitrogen | A32723 | AB_2633275 |
| Alexa488-conjugated goat-anti-rabbit antibody | Invitrogen | A32731 | AB_2633280 |
| Alexa555-conjugated goat-anti-rabbit antibody | Invitrogen | A32732 | AB_2633281 |
| anti-AFP | Thermo scientific | RB-365-A1 | AB_59574 |
| anti-α-Smooth Muscle Actin (D4K9N) XP | CST | 19245S | AB_2734735 |
| anti-Dystrophin | Thermo | PA5-32388 | AB_2549858 |
| anti-LIN28A (D1A1A) XP | CST | 8641S | AB_10997528 |
| anti-MYH2 | DSHB | mAb2F7 | AB_1157865 |
| anti-Nanog-XP | CST | 8822S | AB_11217637 |
| anti-Oct-4A (D6C8T) | CST | 83932S | AB_2721046 |
| anti-Sox2 | abcam | ab97959 | AB_2341193 |
| anti-SSEA1(MC480) | CST | 4744s | AB_1264258 |
| anti-TH (H-196) | SANTA CRUZ | sc-14007 | AB_671397 |
| Alkaline Phosphatase Live Stain (500x) | Thermo | A14353 | |
| Blasticidin S | Sigma-Aldrich | 203350 | |
| BsmBI/Esp3I | NEB | R0580L/R0734L | |
| Carbenicillin | Millipore | 205805-250MG | |
| Collagenase IV | Worthington Biochemical Corporation | LS004189 | |
| Competent Cells | TakaRa | 636763 | |
| CutSmart | NEB | B7204S | |
| CytoTune-iPS 2.0 Sendai Reprogramming Kit | Thermo | A16517 | |
| DirectPCR Lysis Reagent (cell) | VIAGEN BIOTECH | 302-C | |
| Dispase (1 U/mL) | STEMCELL Technologies | 7923 | |
| Doxycycline Hydrochloride | Fisher BioReagents | BP26535 | |
| EcoRI-HF | NEB | R3101L | |
| Fibronectin bovine plasma | SIGMA | F1141 | |
| QIAEX II Gel Extraction Kit (500) | QIAGEN | 20051 | |
| Gelatin from porcine skin, type A | SIGMA | G1890 | |
| HardSet Antifade Mounting Medium with DAPI | Vector | H-1500 | |
| Hygromycin B (50 mg/mL) | Invitrogen | 10687010 | |
| Ketamine HCL Injection | HENRY SCHEIN ANIMAL HEALTH | 45822 | |
| KpnI-HF | NEB | R3142L | |
| lenti-CRISPRv2-blast | Addgene | 83480 | |
| lenti-Guide-Hygro-iRFP670 | Addgene | 99377 | |
| Lipofectamin 3000 Transfection Kit | Invitrogen | L3000015 | |
| LV-TRE-VP64-mouse MyoD-T2A-dsRedExpress2 | Addgene | 60625 | |
| LV-TRE-VP16 mouse MyoD-T2A-dsRedExpress2 | Addgene | 60626 | |
| Mouse on Mouse (M.O.M.) Basic Kit | Vector | BMK-2202 | |
| NotI-HF | NEB | R3189L | |
| Opti-MEM I Reduced Serum Media | ThermoFisher | 31985070 | |
| Polyethylene glycol 4,000 | Alfa Aesar | AAA161510B | |
| Polybrene | SIGMA | TR1003 | |
| Corning BioCoat Poly-D-Lysine/Laminin Culture Slide | CORNING | CB354688 | |
| PowerUp SYBR Green Master Mix | ThermoFisher | A25742 | |
| PrimeSTAR Max Premix | TakaRa | R045 | |
| Proteinase K | VIAGEN BIOTECH | 507-PKP | |
| Puromycin Dihydrochloride | MP Biomedicals | ICN19453980 | |
| qPCR Lentivirus Titration Kit | abm | LV900 | |
| Quick ligation kit | NEB | M2200S | |
| QIAprep Spin Miniprep Kit (250) | QIAGEN | 27106 | |
| QIAGEN Plasmid Plus Midi Kit (100) | QIAGEN | 12945 | |
| RevertAid RT Reverse Transcription Kit | Thermo scientific | K1691 | |
| RNAzol RT | Molecular Research Center, INC | RN 190 | |
| T4 DNA Ligase Reaction Buffer | NEB | B0202S | |
| T4 Polynucleotide Kinase | NEB | M0201S | |
| Terrific Broth Modified | Fisher BioReagents | BP9729-600 | |
| ViralBoost Reagent (500x) | ALSTEM | VB100 |
References
- Mendell, J. R., et al. Evidence-based path to newborn screening for Duchenne muscular dystrophy. Annals of Neurology. 71 (3), 304-313 (2012).
- Batchelor, C. L., Winder, S. J. Sparks, signals and shock absorbers: how dystrophin loss causes muscular dystrophy. Trends Cell Biology. 16 (4), 198-205 (2006).
- Gregorevic, P., et al. Systemic delivery of genes to striated muscles using adeno-associated viral vectors. Nature Medicine. 10 (8), 828-834 (2004).
- Bengtsson, N. E., Seto, J. T., Hall, J. K., Chamberlain, J. S., Odom, G. L. Progress and prospects of gene therapy clinical trials for the muscular dystrophies. Human Molecular Genetics. 25 (R1), R9-R17 (2016).
- Tabebordbar, M., et al. In vivo gene editing in dystrophic mouse muscle and muscle stem cells. Science. 351 (6271), 407-411 (2016).
- Long, C., et al. Postnatal genome editing partially restores dystrophin expression in a mouse model of muscular dystrophy. Science. 351 (6271), 400-403 (2016).
- Nelson, C. E., et al. In vivo genome editing improves muscle function in a mouse model of Duchenne muscular dystrophy. Science. 351 (6271), 403-407 (2016).
- Long, C., et al. Prevention of muscular dystrophy in mice by CRISPR/Cas9-mediated editing of germline DNA. Science. 345 (6201), 1184-1188 (2014).
- El Refaey, M., et al. In Vivo Genome Editing Restores Dystrophin Expression and Cardiac Function in Dystrophic Mice. Circulation Research. 121 (8), 923-929 (2017).
- Amoasii, L., et al. Gene editing restores dystrophin expression in a canine model of Duchenne muscular dystrophy. Science. 362 (6410), 86-91 (2018).
- Eisen, B., et al. Electrophysiological abnormalities in induced pluripotent stem cell-derived cardiomyocytes generated from Duchenne muscular dystrophy patients. Journal of Cellular and Molecular Medicine. 23 (3), 2125-2135 (2019).
- Marion, R. M., et al. Telomeres acquire embryonic stem cell characteristics in induced pluripotent stem cells. Cell Stem Cell. 4 (2), 141-154 (2009).
- Dumont, N. A., et al. Dystrophin expression in muscle stem cells regulates their polarity and asymmetric division. Nature Medicine. 21 (12), 1455-1463 (2015).
- Sacco, A., et al. Short telomeres and stem cell exhaustion model Duchenne muscular dystrophy in mdx/mTR mice. Cell. 143 (7), 1059-1071 (2010).
- Su, X., et al. Purification and Transplantation of Myogenic Progenitor Cell Derived Exosomes to Improve Cardiac Function in Duchenne Muscular Dystrophic Mice. Journal of Visualized Experiments. (146), (2019).
- Su, X., et al. Exosome-Derived Dystrophin from Allograft Myogenic Progenitors Improves Cardiac Function in Duchenne Muscular Dystrophic Mice. Journal of Cardiovascular Translational Research. 11 (5), 412-419 (2018).
- Ousterout, D. G., et al. Multiplex CRISPR/Cas9-based genome editing for correction of dystrophin mutations that cause Duchenne muscular dystrophy. Nature Communications. 6, 6244(2015).
- Barde, I., et al. Efficient control of gene expression in the hematopoietic system using a single Tet-on inducible lentiviral vector. Molecular Therapy. 13 (2), 382-390 (2006).
- Glass, K. A., et al. Tissue-engineered cartilage with inducible and tunable immunomodulatory properties. Biomaterials. 35 (22), 5921-5931 (2014).
Access restricted. Please log in or start a trial to view this content.
Reprints and Permissions
