We investigated skeletal muscle tissue in Bos indicus and crossbred bulls to explain differences in meat quality traits. Warner-Bratzler shear force (WBSF) was found to range from 4.7 kg to 4.2 kg. Myosin heavy chain isoforms revealed differences between animals, and myofibril fragmentation index provided further insights into tenderness (WBSF) variations.
Method Article
Exploring the Longissimus Muscle: Unraveling its Correlation with Meat Quality in Bos indicus and Crossbred Bulls
In This Article
Summary
Abstract
This study investigated muscle tissue in Bos indicus and crossbred bulls to explain differences in meat quality traits. Carcass traits, meat quality parameters, and biochemical and molecular investigations of myofibrillar proteins are described. Methods for evaluating pH, intramuscular fat (IMF), meat color (L*, a*, b*), water losses, tenderness, and molecular biology assays have been outlined. Specific procedures detailing calibration, sample preparation, and data analysis for each method are described. These include techniques such as infrared spectroscopy for IMF content, objective tenderness assessment, and electrophoretic separation of MyHC isoforms.
Color parameters were highlighted as potential tools for predicting beef tenderness, a crucial quality trait influencing consumer decisions. The study employed the Warner-Bratzler shear force (WBSF) method, revealing values of 4.68 and 4.23 kg for Nellore and Angus-Nellore (P < 0.01), respectively. Total cooking losses and biochemical analyses, including myofibril fragmentation index (MFI), provided insights into tenderness variations. Muscle fiber types, particularly myosin heavy chain (MyHC) isoforms, were investigated, with a notable absence of MyHC-IIb isoform in the studied Zebu animals. The relationship between MyHC-I and meat tenderness revealed divergent findings in the literature, highlighting the complexity of this association. Overall, the study provides comprehensive insights into the factors influencing meat quality in Bos indicus and crossbred (Bos taurus × Bos indicus) bulls, offering valuable information for the beef industry.
Introduction
Brazil has the largest commercial cattle herd globally, numbering approximately 220 million animals and ranking as the second-largest meat producer, yielding over 9 million metric tons of carcass equivalent annually1. The beef cattle production sector significantly contributes to the national agricultural system, with total annual sales surpassing R$ 55 billion. Since 2004, Brazil has been a key player in the global meat trade, exporting to over 180 countries, which represents ~50% of the world meat trade2.
Meat tenderness stands out as the paramount quality attribute influencing consumer satisfaction and meat consumption3. By employing biochemical and objective methods to measure meat tenderness, researchers aim to provide valuable insights into factors such as animal genetics, processing techniques, and storage conditions, ultimately enhancing the quality and consistency of meat products for consumers. Such information is useful because meat tenderness has gained increased importance in consumer decision-making during purchases. Moreover, meat tenderness assessment provides valuable information for quality control in meat production and processing industries. By consistently monitoring tenderness, producers can ensure that meat products meet desired standards and specifications. In this context, Brazilian beef cattle producers are progressively embracing intensive feedlot systems with crossbred animals to enhance capital turnover. This system accounts for about 10% tons of carcass produced annually in Brazil4,5.
The escalating demand for improved meat quality by consumers has prompted beef cattle producers to crossbreed with European breeds, primarily Aberdeen Angus6. This strategy aims to produce F1 Angus-Nellore hybrids, known for superior performance, desirable carcass traits, and enhanced meat quality compared to pure zebu animals7,8. In the tropical regions of Brazil, it is common practice to utilize non-castrated animals (bulls) of advanced maturity in finishing farms, potentially compromising meat quality attributes such as color, marbling, and tenderness. Notably, a survey reveals that 95% of animals finished in Brazilian feedlots are males, with 73% being Nellore, followed by 22% crossbred animals and 5% other genotypes9,10.
Understanding the biochemical mechanisms underlying meat tenderness is crucial for improving meat quality. One key aspect is postmortem proteolysis, which affects the structural integrity of muscle fibers11. The myofibril fragmentation index (MFI) is a widely used biochemical assay that quantifies the extent of myofibril degradation, providing insights into the tenderness of meat12. The MFI method involves measuring the fragmentation of myofibrillar proteins, which directly correlates with meat tenderness. This assay complements traditional meat quality assessments and offers a deeper understanding of the biochemical processes that contribute to variations in meat tenderness.
In this context, the present study investigated the skeletal muscle of Bos indicus versus crossbred (Bos taurus × Bos indicus) bulls finished in feedlot, aiming to explain differences in meat quality traits.
Protocol
All procedures with animals complied with the ethical research standards established by the Animal Use Ethics Committee (CEUA) of the "Universidade Estadual Paulista Júlio de Mesquita Filho" - UNESP Botucatu Campus, under protocol 0171/2018.
1. Experimental animals
- Finish 30 Nellore bulls (Bos indicus) and 30 F1 Angus-Nellore bulls (Bos taurus × Bos indicus), aged 20-24 months, in a feedlot. House both groups of animals in collective pens measuring 5 m x 6 m with a concrete floor and equipped with shell-type water troughs, accommodating up to five animals per pen. Ensure that all animals belong to the same management group (born and raised on the same farm) and are submitted to the same feedlot period.
NOTE: In this study, the Nellore bulls had an average initial body weight of 370.7 kg while the F1 Angus-Nellore bulls had an average initial body weight of 380.8 ± 17 kg. - Feedlot diet
- Ensure that the finishing diet is comprised of 11.3% roughage (Tifton hay and sugarcane bagasse) and 88.7% concentrates (ground dry corn grain, soybean meal, corn wet distillers' grains, dry corn gluten feed, and mineral core). Feed the animals for 120 days and provide the diets ad libitum twice a day (at 10:00 a.m. and 04:00 p.m.).
- Slaughter
- Register the final body weight (BWf) at the end of the experimental period. Process all animals at a nearby slaughterhouse, adhering to standard inspection procedures. Prior to slaughter, ensure that the animals undergo a minimum 16 h fast, abstaining from both feed and water.
NOTE: F1 Angus-Nellore bulls exhibited a final body weight of 615.09 ± 57.53 kg, while Nellore bulls had a weight of 545.47 ± 11.45 kg.
- Register the final body weight (BWf) at the end of the experimental period. Process all animals at a nearby slaughterhouse, adhering to standard inspection procedures. Prior to slaughter, ensure that the animals undergo a minimum 16 h fast, abstaining from both feed and water.
- Evaluation of carcass traits
- Weigh the beef carcasses initially and then subject them to a cooling period at 2-4 °C for 48 h. Measurements include hot carcass weight (HCW), rib eye area (REA), and backfat thickness (BFT) at the 12th/13th rib interface, as recommended13. Determine the REA using the grid method with a small grid (18 cm x 13 cm) and measure the BFT in millimeters using a caliper.
- Measure the REA in each carcass by using a reticulated grid (the same as used in the USDA Yield Grade classification system), divided into 1 cm² squares with one dot in the middle. Add all squares within the ribeye tracing perimeter and those along the contour of the tracing passing through the middle dot.
- Measure the BFT at a specific position on the assessment site anywhere between the 12th/13th ribs. To determine this position, measure the length of the rib eye; then, starting at the medial border "A", determine a point three quarters of the way along the rib eye and halfway across "B". Take a caliper through this point and at right angles to the specified rib to the interface between the subcutaneous fat and intermuscular fat. Measure the subcutaneous fat by placing the caliper at a right angle to the line of the subcutaneous fat, from the interface point (Supplemental Figure S1).
- Weigh the beef carcasses initially and then subject them to a cooling period at 2-4 °C for 48 h. Measurements include hot carcass weight (HCW), rib eye area (REA), and backfat thickness (BFT) at the 12th/13th rib interface, as recommended13. Determine the REA using the grid method with a small grid (18 cm x 13 cm) and measure the BFT in millimeters using a caliper.
- Sampling
- Sample Longissimus thoracis (LT) from the left half-carcass (portion of ± 12.0 cm of meat), between the 11th and 13th ribs in the cranial direction. In the laboratory, section the meat samples into steaks of 2.54 cm.
- Aging
- Assess the meat quality traits after a 14 day wet-aging period at a temperature of 0-2 °C in a biological oxygen demand (BOD) incubator. Use steaks of 2.54 cm thickness for the analysis of meat color, pH, intramuscular fat, purge loss, water-holding capacity, objective tenderness, and cooking losses. Pack the steaks separately in plastic bags for high vacuum and low oxygen permeability and after the aging time is reached, keep them frozen at -20 °C until the time of analysis. Thaw the beef samples at 4 °C for 24 h and expose them to oxygen for 30 min at 4 °C (blooming time).
2. Meat pH
- Measure the pH of the meat using a digital pH gauge equipped with a penetration probe. Calibrate it with pH 4.0 and 7.0 buffers at a room temperature of 25 °C. Measure the meat pH at three locations of the LT muscle sample. Manually record the data readings and subsequently export the datasheet; calculate the average of the three readings for meat pH.
3. Intramuscular fat
NOTE: Intramuscular fat (IMF) content was determined using near infrared (NIR) spectroscopy14 and by gravimetric method15.
- Remove the subcutaneous fat from the LT muscle using a scalpel. Then, grind and homogenize the steak for 5 min using a mixer, incorporating approximately 180 g of the sample. Place the sample in a cup, position it inside the sample chamber, and perform subscanning of various zones of the test sample by rotating the sample cup; merge the zones for the final result.
- Take three readings for each sample. After homogenization, place the samples in the plate for subsequent reading. Set the apparatus to NIR transmission, with a moving grating monochromator scanning the region from 850 nm to 1050 nm.
- Export the data sheet and then calculate the average three reading for the IMF. Express the results as a percentage, using the formula: [(IMF average ÷ sample weight) × 100].
- Combine homogenize the LT muscle samples (3.0 g) with a chloroform/methanol methanol/chloroform (2:1) solution for 2 min and subject them to centrifugation (700 × g; 10 min; 20 °C) to segregate the hydrophilic (upper), solid (middle), and hydrophobic (lower) phases.
- Filter the hydrophobic phase obtained post centrifugation using a filter paper on a funnel with slight suction. Transfer the filtrate (bottom phase; lipids in chloroform) to a flask labeled as lipid phase and transfer at least 5 mm of filtrate to a preweighed beaker flask after letting it stand for a few minutes. Then, record the volume of the chloroform layer (at least 150 mL) and aspirate the alcoholic layer.
- Homogenize 100 g aliquots of the sample of fresh or frozen tissue for 2 min with a mixture of 100 mL of chloroform and 200 mL of methanol. Add 100 mL of chloroform to the mixture, blend for 30 s, add 100 mL of distilled water, and blend for another 30 s.
- Filter the homogenate through filter paper on a funnel with slight suction. Apply pressure with the bottom of a beaker when the residue becomes dry to ensure maximum recovery of solvent.
- Transfer the filtrate to a 500 mL graduated cylinder and let it stand for a few minutes to allow separation and clarification. Record the volume of the chloroform layer (at least 150 mL) and aspirate the alcoholic layer.
- Be sure to completely remove the top layer; the chloroform layer contains the purified lipid. For quantitative lipid extraction, recover the lipid trapped in the tissue residue by blending the residue and filter paper with 100 mL of chloroform.
- Filter the mixture through the funnel and rinse the blender jar and residue with a total of 50 mL of chloroform. Mix this filtrate with the original filtrate before removing the alcoholic layer.
NOTE: Filtration is typically rapid; apply pressure with the bottom of a beaker on the dry residue to ensure maximum recovery of solvent.
- Dry the samples in an oven, cool them in a desiccator for at least 24 h, place them in an oven at 110 °C until complete solvent evaporation, further cool them in a desiccator overnight, and finally reweigh them.
- Determine the IMF content by calculating the difference between the initial and final weights of the beaker.
4. Meat color
- Calibrate the device using a black and a white standard plate. Place the white calibration plate near the middle of the plate. When doing a calibration, use the area near the middle of the plate. Calibration is complete after the lamp flashes three times.
- Take measurements after 30 min at 4 °C (blooming time). Obtain color readings from three different locations on the LT muscle sample, carefully avoiding connective tissue and fat.
- At room temperature (20 °C), compute an average from these measurements, as recommended16.
5. Water losses
- Assess purge loss (PL) for all samples. Determine the PL of beef loin sections by measuring the variance between the initial weight before freezing and the final weight after freezing/thawing.
NOTE: Do not evaluate the PL of never-frozen control beef loins. - Gauge the water-holding capacity (WHC) by the weight difference of a meat sample (approximately 1.0 g) before and after being subjected to a pressure of 10 kg for 5 min17.
6. Objective meat tenderness
NOTE: The measurement of Warner-Bratzler shear force (WBSF) was conducted as described18,19.
- Position samples on a grid attached to a glass refractory and cook them in an industrial electric oven until reaching a final temperature of 71 °C. After cooking, cool, weigh, and refrigerate the samples at 4 °C for 24 h.
- Determine cooking losses (CL) using the formula
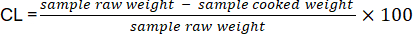 .
- Determine drip loss by weighing the refractory before and after cooking the sample. To this end, place the samples on a grid over a glass refractory to allow drainage of meat juices and fat during cooking.
- Determine evaporation loss by weighing only the sample before and after cooking.
- Record raw and cooked weights and calculate the percentage of DL as the weight of drip after cooking divided by the weight of the thawed meat sample.
- Calculate the evaporation loss percentage (EVP) using the formula [100 - (weight after cooking) ÷ raw weight × 100].
- For the determination of WBSF, section eight cores with a diameter of 1.27 cm using a texture analyzer, equipped with a 3.07 mm Warner-Bratzler Shear Force blade and a V-shaped (60° angle) cutting edge.
- Report the results as the average of six values per sample, in kilograms (kg), after excluding the low and high extremes19.
7. Biochemical assay
NOTE: Postmortem proteolysis was assessed by estimating the myofibril fragmentation index (MFI), following the original procedure outlined by Culler et al.20 and adapted for Bos indicus cattle by Borges et al.21.
- Homogenize fragments of approximately 3 g of LT samples (fat-stripped muscle tissue and connective tissue) in a buffer solution containing 100 mM potassium chloride, 20 mM potassium phosphate at pH 7, 1 mM ethylenediaminetetraacetic acid (EDTA), 1 mM magnesium chloride, and 1 mM sodium azide at 2 °C, followed by centrifugation (1,000 × g for 15 min at 4 °C).
- Resuspend the sediment in 10 volumes (v/w) of isolating medium using a stir rod, then sediment it again at 1,000 × g for 15 min and decant the supernatant.
- Resuspend the sediment in 2.5 volumes (v/w) of isolating medium and separate the connective tissue and debris by passing it through a polyethylene strainer (18 mesh). Use an additional 2.5 volumes (v/w) to allow the myofibrils to pass through the strainer.
- Determine the protein concentration of the suspension of myofibrils using the biuret method of Gornall et al.22. Dilute an aliquot of the myofibril suspension with isolating medium to a protein concentration of 0.5 ± 0.05 mg/mL.
- Immediately measure the absorbance of this suspension at 540 nm. Determine MFI using spectrophotometry at 540 nm. Multiply the absorbance by 200 to obtain the MFI for each sample (and report it as an index without a measurement unit).
8. Molecular biology assay
NOTE: For the analysis of myosin heavy chain (MyHC), the most abundant protein in bovine skeletal muscle, LT samples from both groups were processed following the protocol described in the literature23,24.
- Achieve electrophoretic separation using a gradient SDS-PAGE gel (7-10%) and a 4% stacking gel. Apply 25 µL of each sample to the gel and run it at 70 V, 28 mA, and 4 °C for 1 h, followed by a run at 180 V, 12 mA, and 4 °C for 29 h.
- Employ two different buffers in the runs: the upper gel buffer comprising glycine, Tris(hydroxymethyl)aminomethane base, sodium dodecyl sulfate (SDS), and distilled water, while the lower gel buffer is identical to the upper buffer, with the addition of mercaptoethanol.
- Stain the gels with Coomassie Blue and capture images using appropriate software.
- Identify MyHC isoforms (MyHC-I, MyHC-IIa, MyHC-IIx/d) based on their molecular weights (223.900, 224.243, and 223.875 kDa, respectively). Conduct semi-quantitative analysis by densitometry of the bands corresponding to each isoform, utilizing appropriate software.
- Employ Rat soleus and Extensor digitorum longus (EDL) muscle as positive controls to classify MyHC isoforms, reserving one well in each gel for loading 40 µL of the processed sample.
- For all data, perform the analysis of variance (ANOVA) by the F test, using the following model:
Yij = µ + ti + Ɛij
where Yij is the observed value of the experimental unit referring to treatment i in repetition j; µ is the general effect of the mean; t is the treatment effect (genetic group), and ε is the experimental error. - Compare the means by using the Student's t-test and adopt P-value < 0.05 as the critical probability.
Results
Table 1 displays the carcass traits of the two genetic groups investigated in this study. Notably, differences were identified (P < 0.01) in HCW, REA, and BFT, with crossbred animals exhibiting greater values, suggesting a heterosis effect.
| Variable¹ | Nellore | F1 Angus x Nellore | SEM | P-value |
| BWfinal, kg | 545.47b | 615.09a | 7.32 | <.0001 |
| HCW, kg | 286.87b | 325.12a | 3.26 | <.0001 |
| REA, cm² | 75.17b | 90.48a | 1.66 | <.0001 |
| BFT, mm | 5.72b | 9.16a | 0.62 | 0.001 |
Table 1: Carcass traits of feedlot-finished Nellore (Bos indicus) and F1 Angus-Nellore (Bos taurus × Bos indicus) bulls. a-b Different lowercase letters indicate differences at P < 0.05. Abbreviations: BW = body weight; HCW = hot carcass weight; REA = ribeye area; BFT = backfat thickness; SEM = standard error of mean.
Comparisons of meat quality traits were also performed (Table 2) and no differences were found for meat pH, redness, PL, EVP, and CL (P > 0.05) between Nellore versus F1 Angus-Nellore bulls. However, crossbred bulls had greater IMF, yellowness, WHC, and MFI than Nellore bulls (P < 0.05). Consequently, meat quality traits of Nellore bulls were negatively impacted in terms of tenderness, with greater WBSF and DL (tougher meat), as well as lower WHC and greater moisture.
| Variable¹ | Nellore | F1 Angus x Nellore | SEM | P-value |
| pH | 5.58 | 5.63 | 0.06 | 0.122 |
| Moisture, % | 74.51 a | 73.65 b | 0.21 | 0.017 |
| IMF NIRS, % | 3.79a | 5.11 b | 0.25 | 0.002 |
| IMF gravimetric method, % | 1.95 a | 3.11 b | 0.34 | 0.005 |
| Lightness (L*) | 31.57 a | 30.98 b | 0.58 | 0.008 |
| Redness (a*) | 14.91 | 15.59 | 0.37 | 0.061 |
| Yellowness (b*) | 5.61 a | 6.19 b | 0.17 | 0.003 |
| Purge loss, % | 23.17 | 21.03 | 1.22 | 0.176 |
| Drip loss, % | 3.96 a | 3.67 b | 0.05 | 0.039 |
| Evaporation loss, % | 22.9 | 24.22 | 1.15 | 0.122 |
| Total cooking loss, % | 26.8 | 28.08 | 1.04 | 0.764 |
| WHC, % | 61.3 | 63.5 | 1.01 | 0.042 |
| WBSF, kg | 4.68 a | 4.23 b | 0.17 | 0.002 |
| MFI | 64.95 a | 81.76 b | 1.54 | 0.005 |
Table 2: Meat quality traits of feedlot-finished Nellore (Bos indicus) and F1 Angus-Nellore (Bos taurus × Bos indicus). a-bDifferent lowercase letters indicate differences at P < 0.05. Abbreviations: IMF = intramuscular fat content; WBSF = Warner-Blatzler shear force; MFI = myofibril fragmentation index; WHC = water-holding capacity.
The differences in meat tenderness can be also associated with differences in MyHC IIa (P < 0.01) between experimental groups (Figure 1). F1 Angus-Nellore bulls exhibited a higher abundance of MyHC IIa compared to Nellore bulls. These findings suggest that, for Nellore animals, a modulation occurred from fast-glycolytic fibers (MyHC IIx) to fast-oxidative glycolytic fibers (MyHC IIa). In contrast, for F1 Angus-Nellore animals, this modulation occurred with less magnitude, showing noticeable hypertrophic growth of fast-glycolytic fibers (MyHC IIx). Thus, the expression of the MyHC-IIa isoforms varied distinctly between these groups.
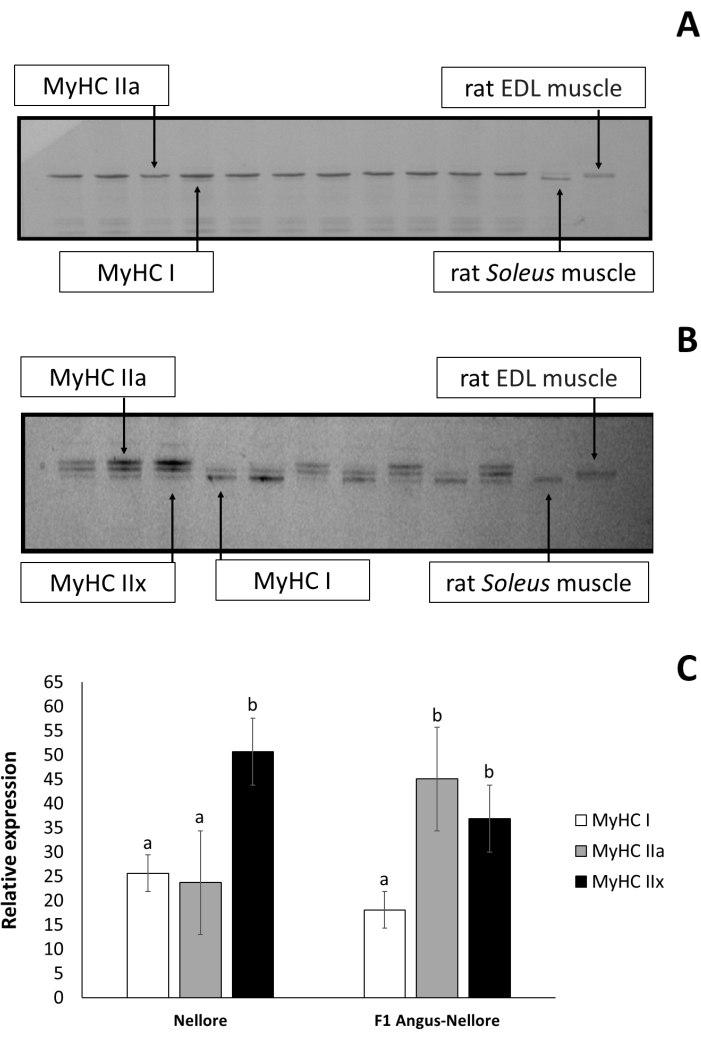
Figure 1: Electrophoresis of myosin heavy chain isoforms of the Longissimus thoracis muscle. (A) Nellore and (B) F1 Angus-Nellore bulls. (C) Relative percentage of MyHC isoforms in the Longissimus thoracis muscle of two experimental groups (SDS-PAGE gel 7-10%). Abbreviations: MyHC = myosin heavy chain; SDS-PAGE = sodium dodecylsulfate-polyacrylamide gel electrophoresis. Please click here to view a larger version of this figure.
Supplemental Figure S1: Method for measuring backfat thickness (BFT) at the interface between the subcutaneous fat and intermuscular fat. The process involves identifying specific anatomical landmarks, including the medial border "A" and a point three-quarters along the rib eye and halfway across "B". A caliper is then positioned perpendicular to the specified rib at point B, extending to the interface between the subcutaneous fat and intermuscular fat. Subcutaneous fat thickness is measured by placing the caliper at a right angle to the line of subcutaneous fat from the interface point. Please click here to download this File.
Discussion
During carcass evaluation, it is crucial to accurately measure growth and quality traits following a 48 h cooling period to obtain consistent and comparable data. The two biological models exhibited divergent carcass traits, particularly HCW, REA, and BFT, which are consistent with findings reported in other studies. The average HCW of Nellore bulls aligns with Brazilian market preferences, which prioritize greater meat production per animal unit with less fat content25. Conversely, crossbred cattle (Bos taurus × Bos indicus) have higher carcass weights and greater marbling scores, which yield meat with superior sensory quality. This meets the market demand for beef with elevated added value, as these attributes are associated with premium meat products26.
The obtained average pH values, ranging between 5.3 and 5.5, closely align with the reported literature values for beef27, which typically range of 5.3 to 5.6. The color variables L*, a*, b* are consistent with the average values for beef cattle observed in other studies7,28. These studies reported b*, a*, and L* variables ranging from 4.0 to 7.0, 13 to 16, and 30.0 to 32.0, respectively. In these meat quality assays, sample preparation must be meticulous, involving the proper handling of muscle samples, including a standardized aging process and blooming time before analysis, to ensure uniformity. Calibration and measurement protocols demand that all devices, such as pH meters and colorimeters, are precisely calibrated before use to maintain the integrity of the measurements.
The color of meat results from the interaction of oxygen with myoglobin in muscle, and the concentration of myoglobin appears to be proportional to the size of the animal29. Similar findings were reported by Purchas et al.30 for European animals (Bos taurus), where they observed higher redness and yellowness in meat of fast-growing Angus cattle compared to slow-growing animals. Prior studies have reported the potential utility of color parameters (L*, a*, b*) as a tool for predicting beef tenderness in both European31 and Zebu animals32.
The examination of meat color is pivotal, as it ranks among the primary factors considered by consumers when purchasing meat, alongside considerations of food safety (product origin and trade), cut type and size, as well as fatness and intramuscular fat (marbling). Consequently, to enhance the likelihood of meat being tender and juicy, consumers are advised to assess meat color, cut size, and, notably, marbling or intramuscular and subcutaneous fat33. Nevertheless, it is evident that color exerts the most significant influence on decision-making during the purchase of meat.
The average WBSF value obtained fell within the range of 4.0 to 4.7 kg. Objective tenderness analysis has been widely employed to assess meat tenderness, as it is considered relatively cost-effective and does not necessitate panelists or sensory tests34. Given the subjective nature of consumer evaluations on beef tenderness, which is influenced by IMF35, instrumental methods are crucial for predicting tenderness ratings. Additionally, the sensitivity of certain methods, such as near-infrared spectroscopy, necessitates precise calibration and consistency in sample preparation; any deviation can result in inaccurate readings.
The original concept of the WBSF instrument has undergone some changes since the 60s36. In the context of beef, this method was standardized by Wheeler et al.37. According to the authors, the preparation and cooking of samples must be meticulously controlled: samples are positioned on a grid over a glass refractory and cooked until they reach an internal temperature of 71 °C. After cooking, the samples are cooled, weighed, and refrigerated at 4 °C for 24 h to stabilize them before further analysis. Cooking losses are calculated using formulas for drip loss and evaporation loss, ensuring that the weight changes due to cooking are accurately quantified. The WBSF measurement is a crucial step, involving the sectioning of eight cores per sample, with the average of six shear force values reported after excluding extremes, providing a reliable measure of meat tenderness. The total cooking losses in the current study, represented by the sum of EL and DL, were comparable to those reported in feedlot-finished beef cattle38. Moreover, it is widely accepted that heat-induced changes in connective tissue contribute to a tenderizing effect. Studies have demonstrated the impact of end cooking temperature on tenderness, revealing changes in myofibrillar structure, whereby both tenderness and CL are affected by protein denaturation39,40. Such chemical or molecular events may influence sensory properties due to alterations in WHC.
The observed results concerning CL and WHC align with expectations, as it is well-established that water distribution and availability in muscle play a pivotal role in juiciness, tenderness, and flavor41. Consequently, higher DL and lower WHC lead to tougher and less juicy meat, as observed in this study for Nellore bulls.
Biochemical analyses such as MFI are used as indicator of meat tenderness. The results obtained in the current study confirm that MFI in beef decreases as the WBSF value increases, possibly indicating reduced myofibrillar fragmentation in tougher meat. Thus, MFI serves as an indicator of muscle fiber proteolysis, increasing with decreasing WBSF42. Researchers reported that a higher rate of myofibrillar proteolysis led to increased tenderness in beef43 and lamb44. This biochemical assay for postmortem proteolysis involves the homogenization of LT samples in a specific buffer solution, followed by centrifugation and resuspension, with the protein concentration determined using the biuret method. The MFI is then measured via spectrophotometry, providing an index that reflects the degree of myofibrillar fragmentation. These meticulously controlled steps ensure the integrity and reliability of the data, crucial for evaluating the quality and market value of meat products.
Furthermore, MFI can explain more than 50% of the variation in tenderness in aged meat. When studying different breeds or groups, variations in meat tenderness are not solely dependent on genetic factors. Particularly for the LT muscle, as indicated in this research, tenderness variation is primarily attributed to the proteolysis of myofibrillar proteins and, to a lesser extent, to sarcomere length and connective tissue content45. Nevertheless, the relationship between WBSF and MFI can serve as a valuable tool for detecting issues in meat tenderness caused by postmortem cold storage processes in the meat industry. It is important to note that while our study provides insights into breed-type differences, it does not constitute a comprehensive genetic evaluation due to the sample size and scope of our research.
Molecular analysis requires stringent control of electrophoresis conditions and subsequent analysis of MyHC isoforms to ensure the reliability of protein separation and identification. Adhering to these critical steps ensures the robustness and reproducibility of the study's findings. Muscle fiber type plays a fundamental role in modulating growth and beef tenderness traits. MyHC proteins are the most abundant proteins in bovine muscle46 and are commonly studied for the molecular recognition of fiber types in each muscle. Some MyHC isoforms, such as MyHC-IIx, have been suggested as biomarkers of meat tenderness in Bos taurus47. However, there have been limited studies evaluating the genes encoding MyHC and quantifying their isoforms in Zebu animals (Bos indicus). The absence of the MyHC-IIb isoform in the studied animals aligns with findings reported in studies on the identification and expression of MyHC in the skeletal muscle of adult cattle48. Specifically, in Nellore cattle, previous studies could not detect the presence of the MyHC-IIb isoform by electrophoresis in the LT muscle. This isoform is more common in double-muscle Bos taurus breeds, such as Blonde d'Aquitaine49.
The relationship between muscle fiber type and beef tenderness has been a topic of ongoing debate. Sample variability is a significant factor, as differences in muscle composition and fiber types among animals can lead to inconsistent results. Environmental factors, including diet and handling conditions, also play a crucial role in influencing meat quality traits. These limitations highlight the need for stringent control and standardization throughout the measurement process to ensure reliable and comparable results. Similar to the findings in the present study, a negative effect of MyHC-I on the tenderness of LT muscle has been reported for Charolais cattle50,51. In contrast, other studies have described a positive effect of MyHC-I on meat tenderness in various breeds, including Aubrac, Salers, Limousin, Charolais, Montbéliard, Holstein, and Blonde d'Aquitaine52,53,54. Divergent results found in the literature might be attributed to genotype differences and limitations of the methods used for the separation and identification of this isoform in bovine LT muscle. Besides, different background environments and diets could also impact meat quality and muscle type traits.
Biochemical analyses, particularly the MFI, shed light on post-mortem beef tenderness mechanisms, showing the key role of muscle fiber types, myosin heavy chain isoforms, and their impacts on beef tenderness. The absence of certain MyHC isoforms in Bos indicus cattle is noted, with implications for beef tenderness variation. Overall, the complex interplay of genetic and biochemical factors regulates beef tenderness and highlights the need for further research in this area. The integration of multiple methods such as WBSF measurement, IMF content analysis, and MyHC isoform electrophoresis helps explain variations in meat quality. The detailed protocols described offer precise steps for assessing meat quality, ensuring that the procedures can be accurately replicated or adapted by other researchers. Additionally, the findings offer valuable genetic insights by highlighting significant differences in meat quality traits between Bos indicus and crossbred bulls.
Disclosures
The authors have nothing to disclose. The funders had no role in study design, data collection and analysis, decision to publish, or preparation of the manuscript.
Acknowledgements
This research was funded by FAPESP (grants 2023/05002-3; 2023/02662-2 and 2024/09871-9), CAPES (Finance code 001), CNPq (304158/2022-4), and by PROPE (IEPe-RC grant number 149) of School of Veterinary Medicine and Animal Science, São Paulo State University.
Materials
| Name | Company | Catalog Number | Comments |
|---|---|---|---|
| Acetone | Merk, Darmstadt, Germany | CAS 67-64-1 | 100014 | solutions used for the electrophoretic separations |
| Anti-MYH-1 Antibody | Merk, Darmstadt, Germany | MABT846 | Rat soleus |
| Anti-Myosin antibody | Abcam, Massachusetts, United States | ab37484 | Myosin heavy chain |
| Anti-Myosin-2 (MYH2) Antibody | Merk, Darmstadt, Germany | MABT840 | Extensor digitorum longus (EDL) |
| Biological oxygen demand (BOD) incubator | TECNAL, São Paulo, Brazil | TE-371/240L | Meat aging |
| Chloroform; absolute analytical reagent | Sigma-Aldrich, Missouri, United States | 67-66-3 | Intramuscular fat |
| CIELab system | Konica Minolta Sensing, Tokyo, Japan | CR-400 colorimeter | Meat color |
| Coomassie Blue | Sigma-Aldrich, Missouri, United States | C.I. 42655) | Myosin heavy chain |
| Electric oven | Venâncio Aires, Rio Grande do Sul, Brazil | Meat tenderness | |
| Ethanol | Merk, Darmstadt, Germany | 64-17-5 | solutions used for the electrophoretic separations |
| Ethylenediaminetetraacetic acid | Sigma-Aldrich, Missouri, United States | 60-00-4 | Post-mortem proteolysis |
| Glass flasks | Sigma-Aldrich, Missouri, United States | solutions used for the electrophoretic separations | |
| Glycine | Sigma-Aldrich, Missouri, United States | G6761 | Myosin heavy chain |
| Infrared spectroscopy - FoodScan | Foss NIRSystems, Madson, United States | FoodScan™ 2 | Intramuscular fat |
| Magnesium chloride | Sigma-Aldrich, Missouri, United States | 7786-30-3 | Post-mortem proteolysis |
| Mercaptoetanol | Sigma-Aldrich, Missouri, United States | M6250 | Myosin heavy chain |
| Methanol, absolute analytical reagent | Sigma-Aldrich, Missouri, United States | 67-56-1 | Intramuscular fat |
| pH meter | LineLab, São Paulo, Brazil | AKLA 71980 | Meat pH |
| PlusOne 2-D Quant Kit | GE Healthcare Product | Code 80-6483-56 | Post-mortem proteolysis |
| Polypropylene | Sigma-Aldrich, Missouri, United States | solutions used for the electrophoretic separations | |
| Potassium chloride | Sigma-Aldrich, Missouri, United States | 7447-40-7 | Post-mortem proteolysis |
| Potassium phosphate | Sigma-Aldrich, Missouri, United States | P0662 | Post-mortem proteolysis |
| R software | Vienna, Austria | version 3.6.2 | Data analysis |
| Sodium azide | Sigma-Aldrich, Missouri, United States | 26628-22-8 | Post-mortem proteolysis |
| Sodium dodecyl sulfate (SDS) | Sigma-Aldrich, Missouri, United States | 822050 | Myosin heavy chain |
| Spectrophotometer | Perkin Elmer, Shelton, United States | Perkin Elmer Lambda 25 UV/Vis | Post-mortem proteolysis |
| Statistical Analysis System | SAS, Cary, North Carolina, United States | version 9.1, | Data analysis |
| Texture Analyzer | AMETEK Brookfield, Massachusetts, United States | CTX | Meat tenderness |
| Tris(hydroxymethyl)aminomethane | Sigma-Aldrich, Missouri, United States | 77-86-1 | Myosin heavy chain |
| Ultrafreezer | Indrel Scientific, Londrina, Paraná, Brazil. | INDREL IULT 335 D - LCD | Sample storage |
| Ultrapure water | Elga PURELAB Ultra Ionic system | solutions used for the electrophoretic separations | |
| Ultra-Turrax high shear mixer | Marconi – MA102/E, Piracicaba, São Paulo, Brazil | Post-mortem proteolysis |
References
- Nunes, C. L. deC., Pflanzer, S. B., Rezende-de-Souza, J. H., Chizzotti, M. L. Beef production and carcass evaluation in Brazil. Anim Front. 14 (2), 15-20 (2024).
- MAPA. Projeções Do Agronegócio: Brasil 2017/18 a 2027/28 Projeções de Longo Prazo / Ministério Da Agricultura, Pecuária e Abastecimento. Biblioteca Nacional de Agricultura. , BINAGRI. Brasília-DF. (2018).
- Bernués, A., Ripoll, G., Panea, B. Consumer segmentation based on convenience orientation and attitudes towards quality attributes of lamb meat. Food Qual Prefer. 26, 211-220 (2012).
- Andrade, T. S., et al. Perception of consultants, feedlot owners, and packers regarding management and marketing decisions on feedlots: A national survey in Brazil (Part II). Can J Anim Sci. 100 (4), 759-770 (2020).
- de Andrade, T. S., et al. Perception of consultants, feedlot owners, and packers regarding the optimal economic slaughter endpoint in feedlots: A national survey in Brazil (Part I). Can J Anim Sci. 100 (4), 745-758 (2020).
- Santiago, B., et al. Comparison of dental carcass maturity in non-castrated male F1 Angus-Nellore cattle finished in feedlot. Food Sci Anim Resour. 41 (3), 554-562 (2021).
- Miguel, G. Z., et al. Immunocastration improves carcass traits and beef color attributes in Nellore and Nellore×Aberdeen Angus crossbred animals finished in feedlot. Meat Sci. 96 (2), 884-891 (2014).
- Costa, N. V., et al. Carcass and meat quality traits in Nellore and F1 Nellore-Araguaia crosses. Genet Mol Res. 14 (2), 5379-5389 (2015).
- Pinto, A. C. J., Millen, D. D. Nutritional recommendations and management practices adopted by feedlot cattle nutritionists: the 2016 Brazilian survey. Can J Anim Sci. 99 (2), 392-407 (2019).
- Costa Junior, C., et al. Brazilian beef cattle feedlot manure management: A country survey. J Anim Sci. 91 (4), 1811-1818 (2013).
- Huang, C., et al. Proteomics discovery of protein biomarkers linked to meat quality traits in post-mortem muscles: Current trends and future prospects: A review. Trends Food Sci Technol. 105, 416-432 (2020).
- Muniz, M. M. M., et al. Use of gene expression profile to identify potentially relevant transcripts to myofibrillar fragmentation index trait. Funct Integr Genomics. 20, 609-619 (2020).
- Official United States Standards for Grades of Carcass Beef. United States Standards for Grades of Carcass Beef. USDA. , Available from: https://www.ams.usda.gov/sites/default/files/media/CarcassBeefStandard.pdf 1-20 (1997).
- Anderson, S. Determination of fat, moisture, and protein in meat and meat products by using the FOSS FoodScan near-infrared spectrophotometer with FOSS artificial neural network calibration model and associated database: Collaborative study. J AOAC Int. 90 (4), 1073-1083 (2007).
- Bligh, E. G., Dyer, W. J. A rapid method of total lipid extraction. Can J Biochem Physiol. 37 (8), 911-917 (1959).
- Hernández Salueña, B., Sáenz Gamasa, C., Diñeiro Rubial, J. M., Alberdi Odriozola, C. CIELAB color paths during meat shelf life. Meat Sci. 157, 107889(2019).
- Rao, M. V., Gault, N. F. S., Kennedy, S. Variations in water-holding capacity due to changes in the fibre diameter, sarcomere length and connective tissue morphology of some beef muscles under acidic conditions below the ultimate pH. Meat Sci. 26 (1), 19-37 (1989).
- Wheeler, T. L., Koohmaraie, M., Cundiff, L. V., Dikeman, M. E. Effects of cooking and shearing methodology on variation in Warner-Bratzler shear force values in beef. J Anim Sci. 72 (9), 2325-2330 (1994).
- AMSA. Research Guidelines for Cookery, Sensory Evaluation, and Instrumental Tenderness Measurements of Meat. American Meat Science Association Educational Foundation. , (2015).
- Culler, R. D., Parrish, F. C., Smith, G. C., Cross, H. R. Relationship of myofibril fragmentation index to certain chemical, physical and sensory characteristics of bovine longissimus muscle. J Food Sci. 43 (4), 1177-1180 (1978).
- Borges, B. O., et al. Polymorphisms in candidate genes and their association with carcass traits and meat quality in Nellore cattle. Pesqui Agropecu Bras. 49 (5), 364-371 (2014).
- Gornall, A. G., Bardawill, C. J., David, M. M. Determination of serum proteins by means of the biuret reaction. J Biol Chem. 177 (2), 751-766 (1949).
- Chardulo, L. A. L., et al. Gene and protein expression of myosin heavy chain in Nellore cattle comparing growth or meat tenderness traits. Anim Biotechnol. 32 (3), 300-309 (2019).
- Vechetti-Júnior, I. J., et al. NFAT isoforms regulate muscle fiber type transition without altering can during aerobic training. Int J Sports Med. 34 (10), 861-867 (2013).
- Ferraz, J. B. S., de Felício, P. E. Production systems - An example from Brazil. Meat Sci. 84, 238-243 (2010).
- Liang, R. R., et al. Tenderness and sensory attributes of the longissimus lumborum muscles with different quality grades from Chinese fattened yellow crossbred steers. Meat Sci. 112, 52-57 (2016).
- Viljoen, H. F., De Kock, H. L., Webb, E. C. Consumer acceptability of dark, firm and dry (DFD) and normal pH beef steaks. Meat Sci. 61 (2), 181-185 (2002).
- Lopes, L. S. F., et al. Application of the principal component analysis , cluster analysis , and partial least square regression on crossbreed Angus-Nellore bulls feedlot finished. Trop Anim Health Prod. 52 (6), 3655-3664 (2020).
- Oddy, V. H., Harper, G. S., Greenwood, P. L., McDonagh, M. B. Nutritional and developmental effects on the intrinsic properties of muscles as they relate to the eating quality of beef. Aust J Exp Agric. 41 (7), 921-942 (2001).
- Purchas, R. W., Burnham, D. L., Morris, S. T. Effects of growth potential and growth path on tenderness of beef longissimus muscle from bulls and steers. J Anim Sci. 80 (12), 3211-3221 (2002).
- Wulf, D. M., O’Connor, S. F., Tatum, J. D., Smith, G. C. Using objective measures of muscle color to predict beef Longissimus tenderness. J Anim Sci. 75 (3), 684-692 (1997).
- Baldassini, W. A., et al. Meat quality traits of Nellore bulls according to different degrees of backfat thickness: A multivariate approach. Anim Prod Sci. 57 (2), 363-370 (2017).
- Chardulo, L. A. L., Silveira, A. C., Vianello, F. Analytical aspects for tropical meat quality assessment. Food Quality, Safety and Technology. Lima, G. P. P., Vianello, F. , Springer-Verlag Wien. 53-62 (2013).
- Chen, L., Opara, U. L. Texture measurement approaches in fresh and processed foods - A review. Food Research International. 51 (2), 823-835 (2013).
- Luo, L., Guo, D., Zhou, G., Chen, K. An investigation on the relationship among marbling features, physiological age and Warner–Bratzler Shear force of steer longissimus dorsi muscle. J Food Sci Technol. 55 (4), 1569-1574 (2018).
- Essex, E. Objective measurements for texture in foods. J Texture Stud. 1, 19-37 (1969).
- Wheeler, T. L., Koohmaraie, M., Shackelford, S. D. Standardized Warner-Bratzler shear force procedures for meat tenderness measurement. , Available from: https://www.ars.usda.gov/ARSUserFiles/30400510/protocols/shearforceprocedures.pdf (1995).
- Severino, M., et al. Proteomics unveils post-mortem changes in beef muscle proteins and provides insight into variations in meat quality traits of crossbred young steers and heifers raised in feedlot. Int J Mol Sci. 23 (20), 12259(2022).
- Bertola, N. C., Bevilacqua, A. E., Zaritsky, N. E. Heat treatment effect on texture changes and thermal denaturation of proteins in beef muscle. J Food Process Preserv. 18 (1), 31-46 (1994).
- Palka, K., Daun, H. Changes in texture, cooking losses, and myofibrillar structure of bovine M. semitendinosus during heating. Meat Sci. 51 (3), 237-243 (1999).
- Pearce, K. L., Rosenvold, K., Andersen, H. J., Hopkins, D. L. Water distribution and mobility in meat during the conversion of muscle to meat and ageing and the impacts on fresh meat quality attributes - A review. Meat Sci. 89 (2), 111-124 (2011).
- Muniz, M. M. M., et al. Use of gene expression profile to identify potentially relevant transcripts to myofibrillar fragmentation index trait. Funct Integr Genomics. 20 (4), 609-619 (2020).
- Baldassini, W., et al. Meat quality and muscle tissue proteome of crossbred bulls finished under feedlot using wet distiller grains by-product. Foods. 11 (20), 3233(2022).
- della Malva, A., et al. In-depth characterization of myofibrillar muscle proteome changes in lambs fed hazelnut skin by-products. Food Biosci. 53, 102836(2023).
- Koohmaraie, M., Kent, M. P., Shackelford, S. D., Veiseth, E., Wheeler, T. L. Meat tenderness and muscle growth: Is there any relationship. Meat Sci. 62 (3), 345-352 (2002).
- Lefaucheur, L., et al. Muscle characteristics and meat quality traits are affected by divergent selection on residual feed intake in pigs. J Anim Sci. 89 (4), 996-1010 (2011).
- Picard, B., et al. Inverse relationships between biomarkers and beef tenderness according to contractile and metabolic properties of the muscle. J Agric Food Chem. 62 (40), 9808-9818 (2014).
- Chikuni, K., Muroya, S., Nakajima, I. Myosin heavy chain isoforms expressed in bovine skeletal muscles. Meat Sci. 67 (1), 87-94 (2004).
- Picard, B., Cassar-Malek, I. Evidence for expression of IIb myosin heavy chain isoform in some skeletal muscles of Blonde d’Aquitaine bulls. Meat Sci. 82 (1), 30-36 (2009).
- Crouse, J. D., Koohmaraie, M., Seideman, S. D. The relationship of muscle fibre size to tenderness of beef. Meat Sci. 30 (4), 295-302 (1991).
- Zamora, F., et al. Predicting variability of ageing and toughness in beef M. Longissimus lumborum et thoracis. Meat Sci. 43 (3-4), 321-333 (1996).
- Strydom, P. E., Naude, R. T., Smith, M. F., Scholtz, M. M., Van Wyk, J. B. Characterisation of indigenous African cattle breeds in relation to meat quality traits. Meat Sci. 55 (1), 79-88 (2000).
- Renand, G., Picard, B., Touraille, C., Berge, P., Lepetit, J. Relationships between muscle characteristics and meat quality traits of young Charolais bulls. Meat Sci. 59 (1), 49-60 (2001).
- Chriki, S., et al. Meta-analysis of the comparison of the metabolic and contractile characteristics of two bovine muscles: Longissimus thoracis and semitendinosus. Meat Sci. 91 (4), 423-429 (2012).
Reprints and Permissions
