Here, we outline a thorough procedure for measuring social recognition between novel, short-term, and long-term relationships using a Four Cups behavioral experimental paradigm. We outline the benefits and potential uses of this paradigm, along with important information for accurately interpreting the outcomes.
Method Article
Paradigm for Social Recognition in Mice for Distinguishing Short- and Long-Term Relationships
In This Article
Summary
Abstract
Social memory is the ability to remember and recognize conspecifics. It is a fundamental aspect of mammalian behavior, with demonstrated survival advantages in highly sociable mammals such as mice and humans. Rodents, particularly mice, are an established animal model extensively used to study social memory and its underlying mechanisms. Most existing social memory paradigms primarily assess short-term social recognition, wherein the relationship duration and familiarity level between the subject and an agent is between 5–15 min. Therefore, existing paradigms and past studies do not capture social memories from long-term relationships and focus on the novelty vs. short-term familiarity dichotomy, leaving a large gap in our mechanistic understanding of social memories. To fill this gap, we designed a simple assay that captures mouse responses to varying levels of familiarity, placing complex social memory recall in an observable, quantifiable context. In the four cups paradigm, a subject mouse freely explores an arena containing four perforated cups placed in each corner. These cups house three agent mice of varying familiarity levels (social stimuli): a long-term familiar (cagemate; 1 month co-housing), a short-term familiar (10 min of prior exposure), a novel conspecific, and an empty cup as a control. CD-1 male mice show a preference for investigating the novel and long-term familiar mouse over investigating short-term familiar mice in this paradigm. This task demonstrates recognition of familiarity level and minimizes aggressive behaviors while still controlling for exposure history. This novel assay provides a platform for directly comparing the neural mechanisms of social memory across long-term, short-term, and novel individuals. The four cups paradigm serves as a novel measurement for long-term familiarity recognition that will complement existing short-term recognition assays.
Introduction
Social memory is a core feature of mammalian social behavior and is particularly well developed in highly social species such as mice and humans. In rodents, recognition of others underlies behavioral dynamics critical for survival within family and conspecific units, including group cohesion, dominance hierarchies, mating behaviors, and parental care1,2. In addition to its evolutionarily advantageous role in animal survival, social memory disruption in humans is a pervasive hallmark across multiple neuropsychiatric and neurological disorders, including autism spectrum disorder, schizophrenia, and Alzheimer's disease3,4,5,6. Because social recognition is fundamental to the daily functioning of social species and has clear clinical importance, developing behavioral assays that accurately capture its multidimensional nature and neural underpinnings is vital. While existing paradigms measure some aspects of social recognition in mice, most assays are designed to assess novelty preferences by comparing novel versus short-term relationships formed over minutes or hours, rather than quantifying recognition of long-term social relationships.
Existing approaches, such as the three-chamber paradigm or the habituation-dishabituation paradigms, assess novelty preference following only brief prior exposure, often limited to 5–15 minutes7,8,9,10,11. These methods have provided substantial insight into the neural mechanisms of these short-term social memories in mice12,13. However, naturalistic social memories and social function must incorporate the distinct mechanisms at play in long-term relationships, built via cohabitation, long-term social hierarchies, or mating partners. While some studies do use the three-chamber paradigm with littermates14 or familiar mice co-housed with the subject for up to 72 h15,16, the paradigm's primary use still focuses on the simple novel vs. familiar dichotomy. This limits comparisons across multiple different familiar mice. With established social recognition paradigms biased towards studying short-term relationships, we identify a clear gap in our knowledge of the neural mechanisms underlying social recognition of long-term relationships.
To address this limitation, we developed the four cups paradigm: a simple, flexible assay designed to differentiate recognition of multiple social familiarity levels within a single testing session. In this paradigm, a subject mouse explores four corners of an open arena, each containing a perforated cup holding a conspecific or a control empty cup. The cups contain a long-term familiar conspecific (cagemate), a short-term familiar conspecific with limited prior exposure (10 min), a novel mouse, and an empty control. Investigation time serves as a quantitative index of social recognition and social preference. This configuration allows simultaneous comparisons across familiarity levels while minimizing direct physical interaction and potential aggressive encounters.
Protocol
All procedures involving animals must be performed in accordance with institutional guidelines and approved by the University of Florida Institutional Animal Care and Use Committee (IACUC).
1. Animal preparation and housing
- Use adult same-sex group-housed mice for all experiments. Handle mice for at least 2 days to habituate to handling and decrease anxiety prior to experimental testing.
- House the mice in standard laboratory cages under a reverse light-dark cycle with ad libitum access to food and water.
NOTE: Adult CD-1 and C57BL/6 mice (3–4 months of age) were used for representative experiments. Mice were housed in groups of 3–4 animals per cage. Representative datasets included 10 male CD-1 mice, 12 female CD-1 mice, and 31 male C57BL/6 mice. The behavior should be run in the subject's active phase (dark phase). Mice included in this study ran between 9 am–6 pm and were kept in a reverse light-dark cycle (dark phase at 8 am–8 pm). - Define a long-term familiar agent as a same-strain and same-sex cagemate that has cohabited with the subject mouse in the same cage for a minimum of 3–4 weeks prior to testing.
- Select short-term familiar and novel conspecific agents from the same strain and sex as the subject mouse.
- Ensure that novel mice have had no prior physical or olfactory exposure to the subject mouse.
- Select a novel agent and a short-term familiar agent from different home cages to avoid similar olfactory cues in those two agents.
NOTE: Record approximate ages for all animals used and minimize reusing the same novel and short-term agents multiple times a day. If the agents are to be reused, provide >2 h of break in homecage between test trials to avoid stressed agents.
2. Arena setup
- Place a clean, square open-field arena (49.5 cm x 49.5 cm x 49.5 cm; Table of Materials) in a quiet behavioral testing room.
- Illuminate the area using a single tall or overhead lamp adjusted to approximately 8–20 lux.
- Place four identically weighed perforated plastic cups in each corner of the arena (Figure 1A).
- Use visually identical cups whenever possible. If different colored cups are used, counterbalance cup assignments and locations across trials.
- Press two sides of each cup flush against the arena walls to restrict access, minimizing hiding behavior and standardizing investigatory angles.
- Use cups that are sufficiently heavy to prevent escape and sufficiently tall to prevent climbing.
NOTE: In this study, the representative data cups and agent location were pseudorandomized across subjects by rotating the colored, plastic cups clockwise while agent type was moved counterclockwise across trials.
- Place the camera high enough that the entire assay box is in frame to avoid blind spots during behavioral coding. Maintain minimal glare and consistent illumination across the box floor (Figure 1A).
- Clean the arena floor and cups thoroughly between trials using an appropriate disinfectant, followed by water to remove residual odors.
- Allow the arena to dry completely before reintroducing animals.
3. Habituation to arena on Day 0
- Place the subject and its cagemates into the arena containing four empty perforated cups and allow free exploration for 20 min.
NOTE: Habituate subjects individually for tethered experiments. Additional habituation sessions may be required. It is recommended to conduct multiple habituation days if mice do not fully explore the entire arena after one day. - Remove all mice from the arena and return to the home cage.
- Place all social agents under cups for 10 min to habituate them to being restrained. Habituate agents from the same home cage simultaneously, one per cup (Figure 1B).
- Clean the arena and cups prior to introducing mice from a new home cage.
NOTE: Allow mice to rest for at least 15 min after transport to the room before beginning the session.
4. Baseline
- Set up the arena according to section 2. Maintain the same arena configuration across all experimental days.
- Place the subject into the arena containing four empty cups and allow free exploration for 10 min.
NOTE: Do not pause the recording at any time, allowing it to continuously record throughout all stages of the current trial.
5. Short-term acquisition
- Use a weighted perforated cup to confine the subject while placing the designated "short-term familiar" agent. Alternatively, expose the subject to the short-term agent in a clean cage.
- If choosing to do the arena exposure, confine a designated short-term familiar agent under one perforated cup in the arena, leaving the other three cups empty.
- Release the subject and allow free exploration for 10 min (Figure 1B).
NOTE: If using the method of exposure to a short-term agent in an arena, alternate the corner used for the short-term familiar agent across subjects to avoid spatial bias.
6. Inter-trial interval (ITI)
- Retrieve the short-term familiar agent and place it back in its home cage. Allow the subject mouse to remain alone in the arena and move freely for 10 min.
- Gather novel and long-term familiar agent mice for the test phase.
NOTE: Return the short-term familiar agent to the same cup used during short-term acquisition (section 5). This is recommended to avoid novelty in spatial location if doing short-term acquisition in an arena.
7. Social recognition phase
- Place an additional weighted perforated cup on the subject mouse.
- Place one mouse under each of the three weighted perforated cups: a long-term familiar (cagemate), a short-term familiar, and a novel conspecific. Leave a designated fourth cup empty as a control.
NOTE: Label cup tops to identify agent locations during behavioral scoring. - Remove the perforated cup from the subject mouse in the center of the arena and allow free exploration for 10 min (Figure 1A).
- Remove all mice at the end of the 10 min interval and stop recording.
- Return all mice to their home cages.
- Clean the arena and cups thoroughly before the next trial.
NOTE: Keep replacement cups available in case of damage.
8. Behavioral scoring
- Import all recorded videos into behavioral analysis software capable of manual annotation, such as Behavioral Observation Research Interactive Software (BORIS).
NOTE: Behavioral scoring was not blinded to cagemate location, given that labels with agent ID were located above each cup and visible in the videos, and cage number could be inferred. Scorers were not actively paying attention to visible labels and were blinded to the identity of the novel and short-term agent. All scorers followed predefined operational definitions of investigatory behavior and standardized scoring criteria. - Define the behavioral matrix before scoring.
- Define an investigation bout as the subject mouse positioning its nose within 1 cm of a cup while exhibiting sustained investigatory posture.
NOTE: Include chewing and gnawing directed at the cup as investigation bouts. - Manually annotate the total investigation duration for each cup across the 10-min social recognition test phase. Score baseline and acquisition as desired.
NOTE: Automated pose tracking may be used with a 1 cm semicircular region of interest surrounding each cup. - Export annotated data for subsequent statistical analysis.
Results
Following the four cups paradigm protocol, CD-1 male mice exhibited differential social investigation behavior across the long-term familiar (cagemate), short-term familiar, and novel conspecifics (Figure 2). For each agent, a discrimination index (DI) was calculated based on seconds spent investigating in that agent vs the empty cup, calculated as (agent − empty)/(agent + empty) during the 10-min social recognition phase. This index was normally distributed based on the Shapiro-Wilk test; therefore, we used statistical tests that assume normality of data. Mice exhibited significantly greater discrimination toward the novel conspecific compared to the short-term familiar conspecific (Figure 2; novel vs. short-term t(9) = 3.70, Bonferroni-Holm-adjusted p = 0.01). The paradigm also revealed that mice displayed significantly greater discrimination toward the long-term familiar cagemate compared to the short-term familiar conspecific (Figure 2; cagemate vs. short-term t(9) = 2.87, Bonferroni-Holm-adjusted p = 0.04). There was no significant difference in discrimination between the novel conspecific and the cagemate (Figure 2; novel vs. cagemate t(9) = -1.13, adjusted p = 0.29), suggesting that mice preferentially investigated both novel and long-term familiar conspecifics over the short-term familiar mouse. Investigation time at each cup location during the empty-arena baseline did not differ based on which social agent would later occupy that specific cup position, confirming that there was not a prior cup preference that resulted in our results (novel baseline vs. cagemate baseline t(9) = -1.99, p = 0.23; novel vs. short-term baseline t(9) = -1.97, p = 0.23; cagemate vs. short-term baseline t(9) = 0.54, p = 0.60).
In contrast, CD-1 female mice did not exhibit significant differences in discrimination index among the novel, short-term familiar, and long-term familiar conspecifics (Figure 3). No significant differences were observed between novel and short-term familiar (p = 0.35), novel and cagemate (p = 0.69), or short-term familiar and cagemate (p = 0.70). Female mice broadly investigated all agents over the empty cup, showing a distinct pattern of behavior in this task, possibly reflecting broader sociability compared to male mice.
Similarly, C57BL/6 male mice exhibited a trend in the same direction, with greater discrimination toward the novel conspecific than toward the short-term familiar conspecific. This difference approached, but did not reach, significance after the Bonferroni-Holm correction, suggesting greater between-subject variance in this larger C57BL/6 cohort (n = 31) than in the CD-1 males (Figure 4; adjusted p = 0.055). No significant differences were observed between the novel and cagemate (p = 0.62) or between the short-term familiar and cagemate (p = 0.62). These results suggest that the strong investigatory behavior of cagemates observed in CD1 males varies across strains and sexes.
To determine whether social dominance contributed to cagemate investigation, urine-marking David scores were correlated with cagemate discrimination index. No significant correlation was observed in either CD-1 male mice (Pearson's r = 0.28, p = 0.44) or C57BL/6 male mice (Pearson's r = 0.10, p = 0.57), suggesting that social rank did not influence the cagemate discrimination index.
Together, these results demonstrate that the four cups paradigm can detect differential social investigation while simultaneously assessing long-term and short-term familiarity, as well as social novelty, within a single behavioral session. Importantly, sex and strain can impact behavior in this assay.
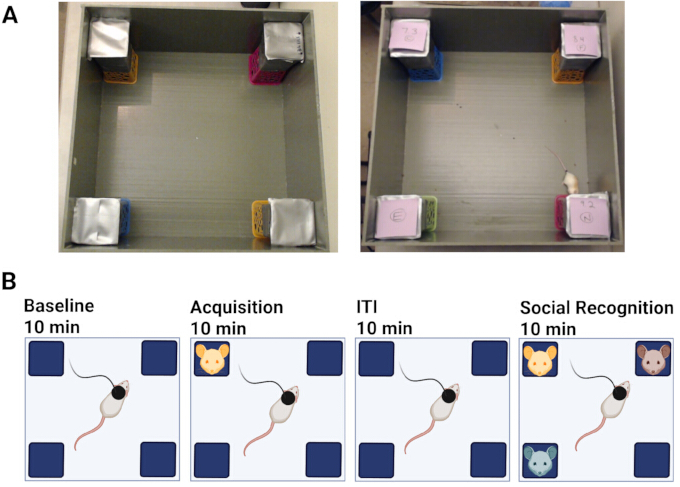
Figure 1: Setup and experimentation process of the four cups paradigm. (A) Left, the four cups paradigm box with four perforated empty cups. Right, subject exploring the four cups paradigm box with four perforated cups with agents in place. Labels indicate social agent identity to facilitate accurate behavioral scoring. (B) Behavioral schematic for Day 1 of the paradigm. Mouse colors indicate agent identities. Note that the images were taken with a camera flash, which makes the appearance of a bright arena compared to the 8–20 lux lighting used for experimentation. Please click here to view a larger version of this figure.
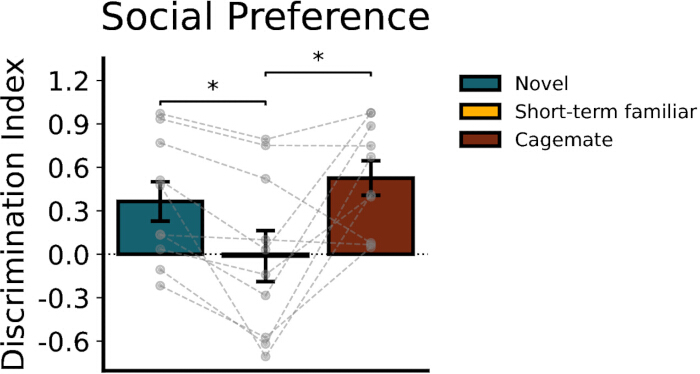
Figure 2: Social preference in the four cups paradigm in CD-1 male Mice. Discrimination index (DI) for investigation of the novel, short-term familiar, and long-term familiar (cagemate) conspecifics during the 10-min social recognition phase. DI was calculated as (agent – empty)/(agent + empty). Mice exhibited significantly greater discrimination towards the novel and cagemate conspecifics compared with the short-term familiar conspecific (p < 0.05), whereas no significant difference was observed between novel and cagemate discrimination. Data are presented as mean ± standard error for 10 mice. Statistical comparisons were performed using paired t-tests with Bonferroni-Holm correction for multiple comparisons. *p < 0.05. Please click here to view a larger version of this figure.
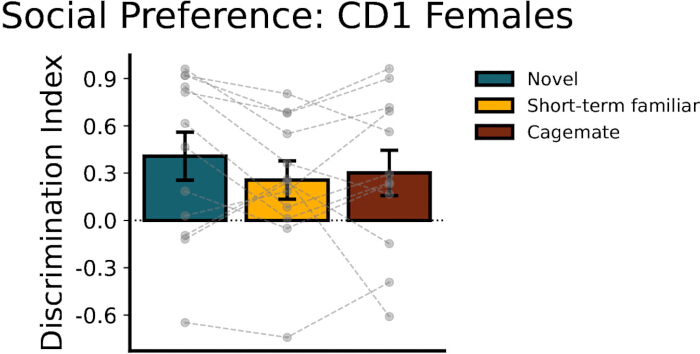
Figure 3: Social preference in the four cups paradigm in CD-1 female Mice. Discrimination index (DI) for investigation of the novel, short-term familiar, and long-term familiar (cagemate) conspecifics during the 10-min social recognition phase. DI was calculated as (agent – empty)/(agent + empty). No significant differences in the discrimination index were observed among the three social stimuli. Data are presented as mean ± standard error of the mean across 12 mice. Statistical comparisons were performed using paired t-tests with Bonferroni-Holm correction for multiple comparisons. *p < 0.05. Please click here to view a larger version of this figure.
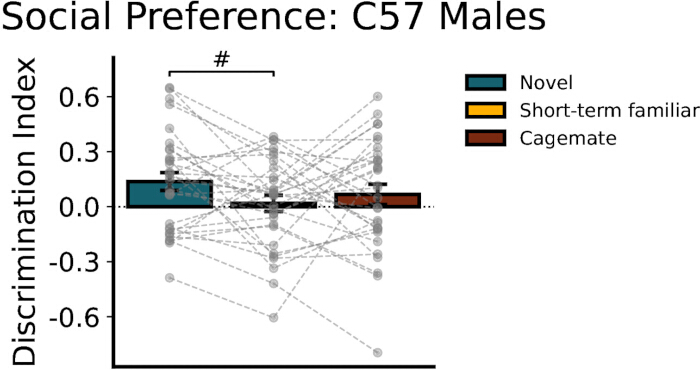
Figure 4: Social preference in the four cups paradigm in C57BL/6 male mice. Discrimination index (DI) for investigation of the novel, short-term familiar, and long-term familiar (cagemate) conspecifics during the 10-min social recognition phase. DI was calculated as (agent − empty)/(agent + empty). A trend toward greater discrimination of the novel conspecific than of the short-term familiar conspecific was observed but did not remain significant after Bonferroni-Holm correction (p = 0.055). No significant differences were observed between novel and cagemate or between short-term familiar and cagemate. Data are presented as mean ± standard error of the mean across 31 mice. Statistical comparisons were performed using paired t-tests with Bonferroni-Holm correction for multiple comparisons. #p < 0.06. Please click here to view a larger version of this figure.
Discussion
There are key considerations for applying the four cups paradigm to effectively and reliably measure these social dynamics in other laboratory settings. Habituation on Day 0 reduces non-social novelty-driven exploration of the arena and cups, which can otherwise mask social investigation during testing7,8,9. Precise control of the short-term familiarization duration is also essential, as small differences in exposure time can significantly alter subsequent preference patterns8,9,10. The 10-min familiarization period was selected to establish a robust short-term social memory while remaining consistent with previously described social recognition paradigms that use brief exposure periods to distinguish familiar from novel conspecifics7,8,10. Additionally, a 3–4 week co-housing period was selected to establish stable long-term social familiarity through prolonged cohabitation rather than repeated brief exposures. This duration provides sufficient opportunity for sustained social interactions and the formation of enduring familiarity between cagemates10. The distinction between the 10-min familiarization period and the 3–4 week co-housing period was intentionally designed to create two qualitatively different levels of familiarity (recent and long-term) within the same behavioral session. During experimentation, counterbalancing agent identities across cup positions across trials is necessary to control for inherent spatial biases in mice7,8. Repeated use of agent mice across trials may alter agent stress levels and, thus, subject investigation behavior. To minimize potential confounds, agent mice were not repeatedly used within a single testing day when possible, and agent identity and cup location were counterbalanced across subjects. In addition, because social dominance has the potential to influence social investigation, dominance hierarchy was assessed using territorial-based dominance and David scores. No significant relationship was observed between David score and cagemate discrimination index in CD-1 male mice and C57BL/6 male mice, suggesting that the observed preference for long-term familiar conspecifics was not explained by dominance status. During analysis, consistent operational definitions of investigatory behaviors, particularly investigation duration, are required to ensure reproducibility across scorers and experimental cohorts. One potential challenge faced by all investigation-based social paradigms is "floor effects", near-zero investigation times that prevent comparisons. For mouse strains that exhibit low levels of social investigation, further reducing visible illumination and using infrared video tracking may reduce anxiety and increase exploratory behavior.
The protocol allows for flexibility and modification depending on experimental goals, but certain adaptations require careful consideration. Cup material is a key variable in the assay. While this protocol uses perforated plastic cups, weighted metal cups with smaller metal perforations may reduce chewing and escape attempts compared to lightweight plastic cups. The use of plastic cups may increase manipulation behaviors, including gnawing or climbing, which should be monitored and annotated during scoring. An alternative approach is to replace the perforated cups with tall, perforated vertical dividers that separate each corner from the central arena while maintaining olfactory and limited visual communication. Although this design may further reduce climbing behavior, removable perforated cups provide the practical advantage of rapidly converting a standard open-field arena into the four cups paradigm without requiring permanent modifications. Excessive interaction with the cups can be mitigated by increasing cup weight, modifying perforation size, and maintaining consistent color to reduce sources of bias. Additionally, agent mice should be counterbalanced and not reused within a single testing day to reduce unintended familiarity effects.
Several limitations of the four cups paradigm should be acknowledged. Because social interaction is restricted by perforated barriers, the assay primarily assesses subject-initiated, non-reciprocal investigation based on olfactory and limited visual cues rather than direct physical contact8,9. Moreover, the use of cups as a physical and visual barrier introduces potential ambiguity in interpreting investigatory behavior. In cases where increased investigation of cagemates is observed, particularly in CD-1 males, it remains unclear whether this reflects just social recognition or a combination of investigation and affiliative motivation, including helping-related behavior toward a familiar conspecific (e.g., attempts to aid cagemate escape by chewing on the plastic cup). These considerations underscore the importance of cautious interpretation and, whenever possible, the use of complementary behavioral assays. Pre-existing social relationships among cagemates, including dominance hierarchy, affiliative interactions, and prior social experiences, may also contribute to investigation preferences. However, we did not observe an apparent relationship between dominance rank and the investigation behavior of cagemates. Nevertheless, these factors may differ across strains, housing conditions, and experimental paradigms and should be considered when interpreting long-term familiarity preferences.
Compared to existing social recognition assays, the four cups paradigm enables the simultaneous comparison of multiple agents, such as a long-term familiar, short-term familiar, and novel conspecific, within a single behavioral session. Traditional paradigms, such as the three-chamber and habituation–dishabituation assays, primarily assess short-term novelty preference following brief exposure periods7,8,9,10. Previous studies have also incorporated long-term cagemates alongside novel conspecifics, including unrestricted social interaction paradigms and modified multi-chamber arenas designed to assess social familiarity17,18. However, these approaches do not simultaneously compare long-term familiar, short-term familiar, and novel social stimuli within the same assay. By incorporating long-term cagemates in tandem with short-term agents, the four cups paradigm provides a means to investigate enduring social memories that arise from extended cohabitation. Representative data from both male and female CD-1 mice demonstrate that the four cups paradigm can be successfully applied across sexes, showcasing sex specific behavioral patterns. Similarly, representative data from both CD-1 and C57BL/6 mice further demonstrate that the four cups paradigm can be successfully implemented across multiple commonly used laboratory strains. Although social recognition and novelty preference often vary across mouse strains7,19, the overall pattern of familiarity discrimination observed in males of both strains suggests that the assay is broadly applicable. Nevertheless, because social recognition behaviors may vary across strain, sex, age, and experimental context, investigators should validate the assay in the specific animal model relevant to their question. Further, while this paradigm could be adapted in a 4-arm or 4-chamber arena, running in an open-field arena allows greater dissociation between navigational and spatial memory and social memory. The spatial memory load is greater when navigating distinct compartments or arms; therefore, for investigating social memory mechanisms, spatial memory should be an important variable to assess. Netser et al (2017) also discuss these caveats regarding the typical 3-chamber assay arena as they propose an analogous two-chamber arena alternative, which minimizes the need for spatial navigation20. This method is well-suited for studies examining the neural representation of social familiarity, longitudinal changes in social cognition, and conditions in which long-term social memory may be selectively altered.
Disclosures
The authors have nothing to disclose.
Acknowledgements
This work was supported by the McKnight Neuroscience Award and the Klingenstein Neuroscience Award to NPC.
Materials
| Name | Company | Catalog Number | Comments |
|---|---|---|---|
| Behavioral Scoring Software | Behavioral Observation Research Interactive Software | Version 9.12.7 | Software for manual event annotation |
| Open-field arena | Rafferty Machine and Tool | Custom made | Structural FRP fiberglass sheet, square arena (49.5 cm x 49.5 cm x 49.5 cm); Non-transparent walls, if arena transparent, cover outside walls with paper to minimize distractions for animal |
| Overhead camera | Logitech | Logitech C920x HD Pro PC Webcam | Camera capable of continuous video recording; Mounted above center of arena |
| Perforated cups | Chinco Store | ONG-Chinco-0279 | dimensions of cups: 4.01"L x 4.01"W x 4.52"H; Perforated plastic or metal cups, could be square or cylindrical |
| Prism | Graph Pad | Version 10.6.0 | Software for data analysis; Could be done with other software |
References
- Wolff JO, Sherman PW, editors. Rodent societies: an ecological and evolutionary perspective. University of Chicago Press; Chicago; 2008.
- Thor DH, Holloway WR. Social memory of the male laboratory rat. J Comp Physiol Psychol. 1982;96(6):1000-1006.
- Theory of mind and autism: A review. International Review of Research in Mental Retardation. Academic Press; 2000.
- Bediou B, et al. Impaired social cognition in mild Alzheimer disease. J Geriatr Psychiatry Neurol. 2009;22(2):130-140.
- Green MF, Horan WP, Lee J. Social cognition in schizophrenia. Nat Rev Neurosci. 2015;16(10):620-631.
- Bäckman L, Herlitz A. The relationship between prior knowledge and face recognition memory in normal aging and Alzheimer's disease. J Gerontol. 1990;45(3):P94-P100.
- Moy SS, et al. Sociability and preference for social novelty in five inbred strains: An approach to assess autistic-like behavior in mice. Genes Brain Behav. 2004;3(5):287-302.
- Engelmann M, Hädicke J, Noack J. Testing declarative memory in laboratory rats and mice using the nonconditioned social discrimination procedure. Nat Protoc. 2011;6(8):1152-1162.
- van der Kooij MA, Sandi C. Social memories in rodents: Methods, mechanisms and modulation by stress. Neurosci Biobehav Rev. 2012;36(7):1763-1772.
- Cum M, et al. A systematic review and meta-analysis of how social memory is studied. Sci Rep. 2024;14(1):2221.
- Oliva A, Fernández-Ruiz A, Leroy F, Siegelbaum SA. Hippocampal CA2 sharp-wave ripples reactivate and promote social memory. Nature. 2020;587(7833):264-269.
- Oliva A. Neuronal ensemble dynamics in social memory. Curr Opin Neurobiol. 2023;78:102654.
- Okuyama T. Social memory engram in the hippocampus. Neurosci Res. 2018;129:17-23.
- Hitti FL, Siegelbaum SA. The hippocampal CA2 region is essential for social memory. Nature. 2014;508(7494):88-92.
- Dykstra B, Kim P, Lin A, Berman GJ, Murugan M. The intermediate CA1 and CA3 subfields of the hippocampus differentially encode social recognition. bioRxiv. 2025; doi.org/10.1101/2025.10.27.684580.
- Rashid M, et al. A ventral hippocampal-lateral septum pathway regulates social novelty preference. eLife. 2025;13:RP97259.
- Phillips ML, Robinson HA, Pozzo-Miller L. Ventral hippocampal projections to the medial prefrontal cortex regulate social memory. eLife. 2019;8:e44182.
- Medeiros D, Polepalli L, Li W, Pozzo-Miller L. Altered activity of mPFC pyramidal neurons and parvalbumin-expressing interneurons during social interactions in a Mecp2 mouse model for Rett syndrome. J Neurophysiol. 2025;134(6):2070-2085.
- Netser S, et al. Distinct dynamics of social motivation drive differential social behavior in laboratory rat and mouse strains. Nat Commun. 2020;11(1):5908.
- Netser S, Haskal S, Magalnik H, Wagner S. A novel system for tracking social preference dynamics in mice reveals sex- and strain-specific characteristics. Mol Autism. 2017;8:53.
Reprints and Permissions
This article has been published
Video Coming Soon